37 A Common Currency
Bodily Need, Allostatic Prediction, and Value-Guided Choice
37.1 Value begins in a regulated body
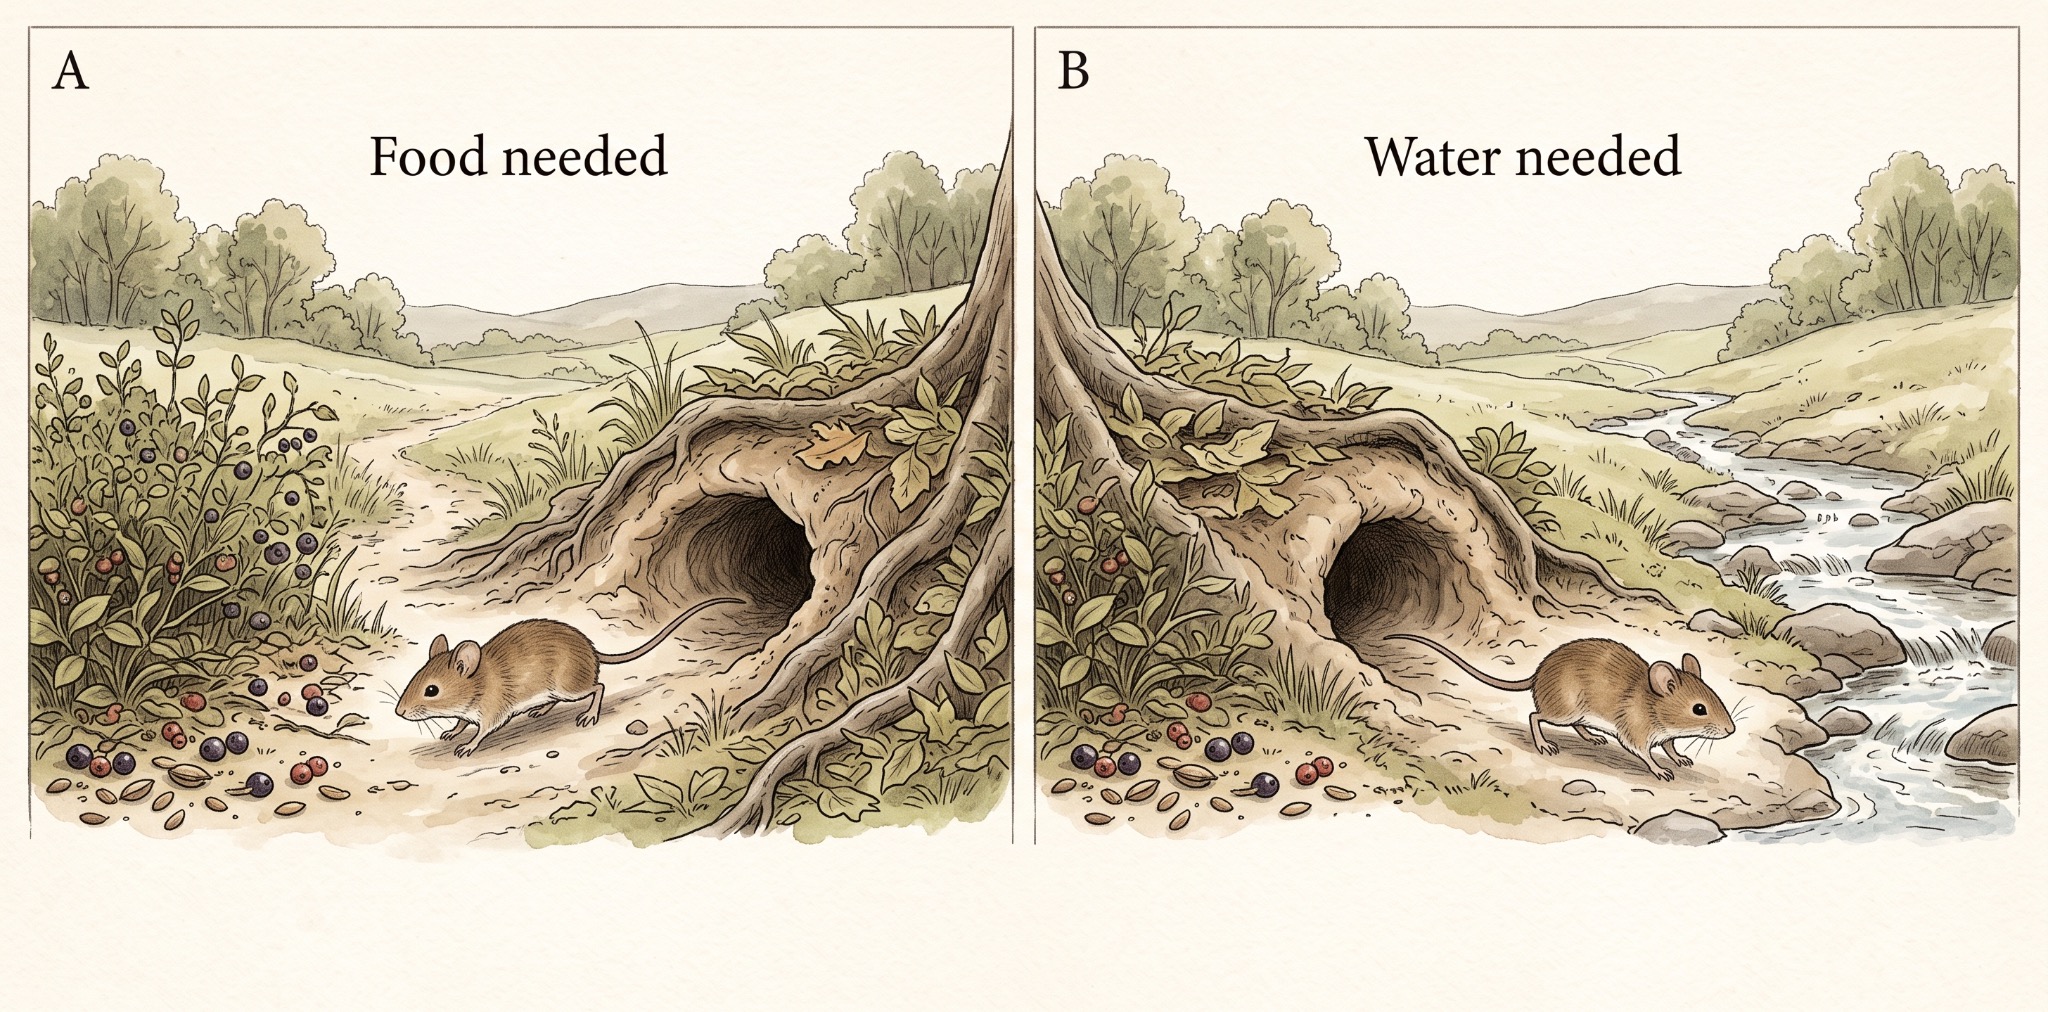
An animal leaving shelter may have food in one direction, water in another, and unfamiliar terrain beyond both. Each possibility offers a different return and imposes different costs. Food supplies energy; water corrects a fluid deficit; shelter reduces exposure; exploration may reveal something useful for a later visit. The animal can sometimes serve several needs together, feeding in shade or investigating while moving toward water. But incompatible routes and movements still compete for the same body, and time spent pursuing one outcome is time unavailable for another. Several predicted consequences must become comparable enough for one course of action to gain control.
This problem is often introduced through economic choice. The biological problem is much older. A vertebrate can be hungry, dehydrated, overheated, injured, threatened, and uncertain about its surroundings at the same time. The consequences of an action depend on that combination of conditions. Water gains value as a fluid deficit grows. Shade becomes worth seeking when continued exposure threatens to overheat the body. A familiar shelter matters more when predation risk rises. Information about another route can justify present effort if the route may be needed later. Economic choice is a special case of an older regulatory problem: different expected consequences compete for control of one body.
Chapter 35 established that consequences alter the competition among actions and that their effects depend on what the organism needs. The present chapter asks how several unlike consequences enter the same choice. Its starting point is that value is a relation between an expected outcome and an organism in a particular state. The object contributes its properties, but those properties acquire significance through what they would do for the organism. Michel Cabanac used the term alliesthesia for the change in pleasantness produced by a change in internal state: warmth can be welcome when cold and oppressive when hot; a food can be attractive when hungry and unappealing after satiety [@cabanac1971pleasure]. The sensory event can remain the same while its significance changes.
The relation can be written compactly as \(V(o \mid s)\): the value of outcome \(o\) conditional on state \(s\). Here, state includes bodily need, current context, recent experience, expected effort, available alternatives, and predictions about the conditions in which the outcome will arrive. A cup of water can have little value after drinking, high value during dehydration, and high anticipatory value before a long crossing through heat. Homeostatic regulation makes an existing deficit consequential. Allostatic regulation allows an expected demand to influence action before that deficit develops.
Human values extend this relation across learning, language, and institutions. Money, a promise, professional achievement, social approval, and knowledge can govern behavior over years. Reducing each of them to a disguised calorie count would explain little. Their significance depends on a history of learning and on the futures they make possible: access to resources, affiliation, obligations, safety, information, and courses of action that would otherwise be unavailable. The position developed here is that this elaboration remains rooted in the problems of an embodied organism. Neural value is the current significance of a consequence within that organism’s ongoing life.
A few distinctions help keep the argument precise. An outcome is an event predicted by an action or cue. A reinforcer is identified by its effect on subsequent behavior or learning. Subjective value concerns how an outcome is currently ranked or weighted in choice; it is often inferred from the choices an organism makes. Pleasure concerns the hedonic quality of experience, while motivation concerns the recruitment and persistence of action. Salience concerns processing priority. A distant water source can be valued before it is tasted. A learned cue can motivate pursuit without being pleasurable itself. A painful stimulus can dominate attention while carrying strongly negative value. These distinctions will matter again when the unit turns to bodily anticipation and the initiation of action.
37.2 Comparable enough to choose
Bodily regulation gives consequences their significance, but it leaves the comparison problem unresolved. How can food, water, shelter, and information influence the same decision when their sensory properties and biological effects differ so much?
The common-currency hypothesis proposes that dissimilar outcomes can be represented in a shared decision format. A value signal that generalizes across the identity of the outcome would allow otherwise unlike options to exert comparable influence on choice. The hypothesis makes a stronger claim than the observation that animals choose: it proposes something about the neural representation through which comparison occurs. Whether a particular task uses such a signal, and where that signal affects the choice, are empirical questions.
The currency metaphor has an immediate limitation. A value of seven says how an option ranks on some scale; by itself, it says nothing about whether the option is water, food, warmth, or social contact. Yet that identity must remain available. Selective satiety should reduce the influence of one food while leaving another relatively attractive. A change in thirst should alter the significance of water. A new obstacle should change the cost of one route without changing the destination. Outcome identity specifies what is expected; decision value expresses how strongly that expected outcome should influence the current choice. Adaptive comparison depends on both.
Delay, uncertainty, and effort likewise remain part of the option. Water ten seconds away and water an hour away are the same kind of outcome but different prospects. A preferred food behind a dangerous barrier may lose to a less attractive food within reach. Decision value can summarize these dimensions for the comparison at hand, provided the information from which the summary was derived remains available for revision. The controller needs a comparison that is general enough to guide action and specific enough to change when circumstances change.
This distinction also separates a mathematical description from a neural explanation. If choices are sufficiently orderly, a utility function can assign numbers that reproduce their ranking. That is a useful description of behavior. It does not establish that the brain explicitly computes that number, or that one region converts every attribute into a universal scale. The physiological question is which quantities neural activity distinguishes, how those quantities depend on state, and whether changing the activity changes the decision.
37.3 An exchange rate in orbitofrontal cortex
An influential experiment by Camillo Padoa-Schioppa and John Assad approached this question by allowing monkeys to choose between two juices offered in varying quantities. The critical first measurement was behavioral. By changing the amounts, the investigators found the indifference point at which the monkey chose either offer about equally often. If one unit of juice A was chosen as often as three units of juice B, the revealed exchange rate was approximately \(1A = 3B\). That ratio made it possible to distinguish physical quantity from subjective equivalence [@padoaschioppaassad2006].
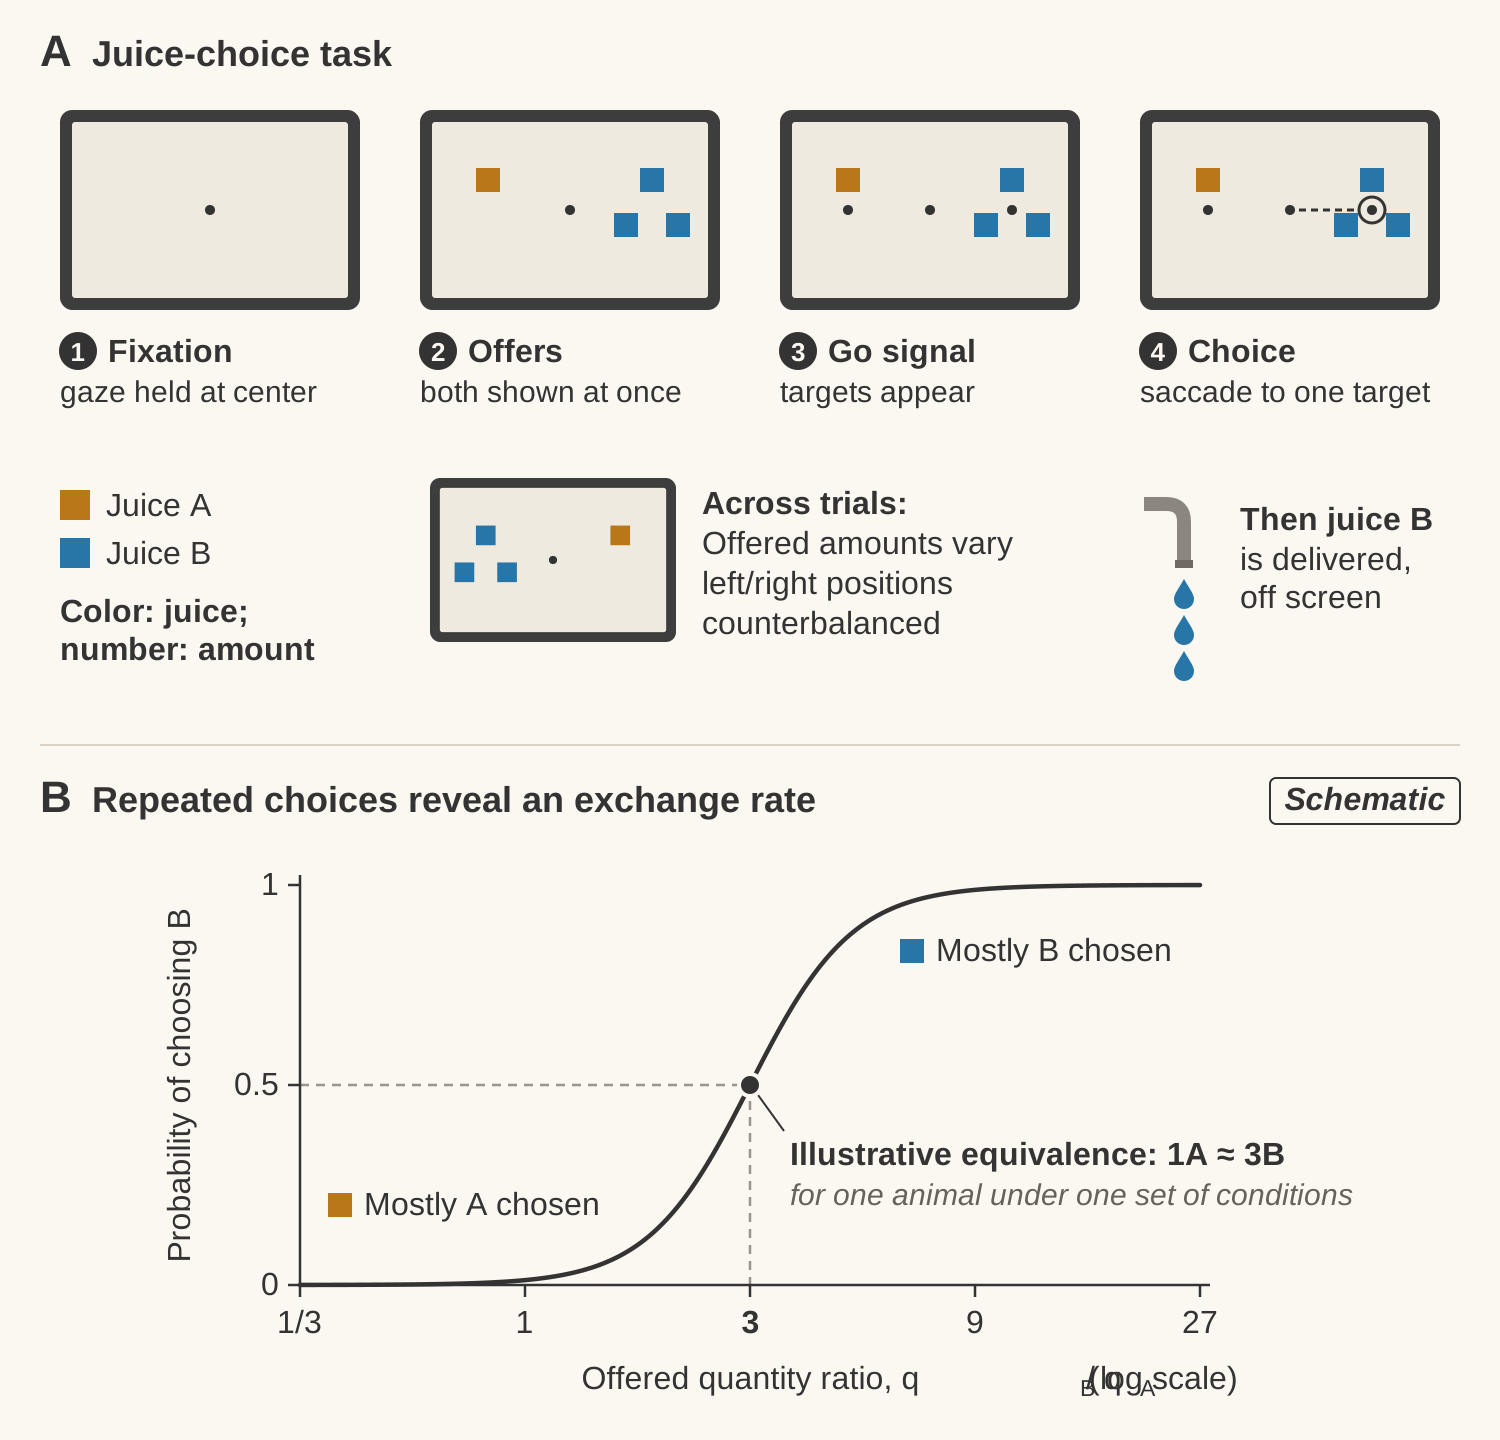
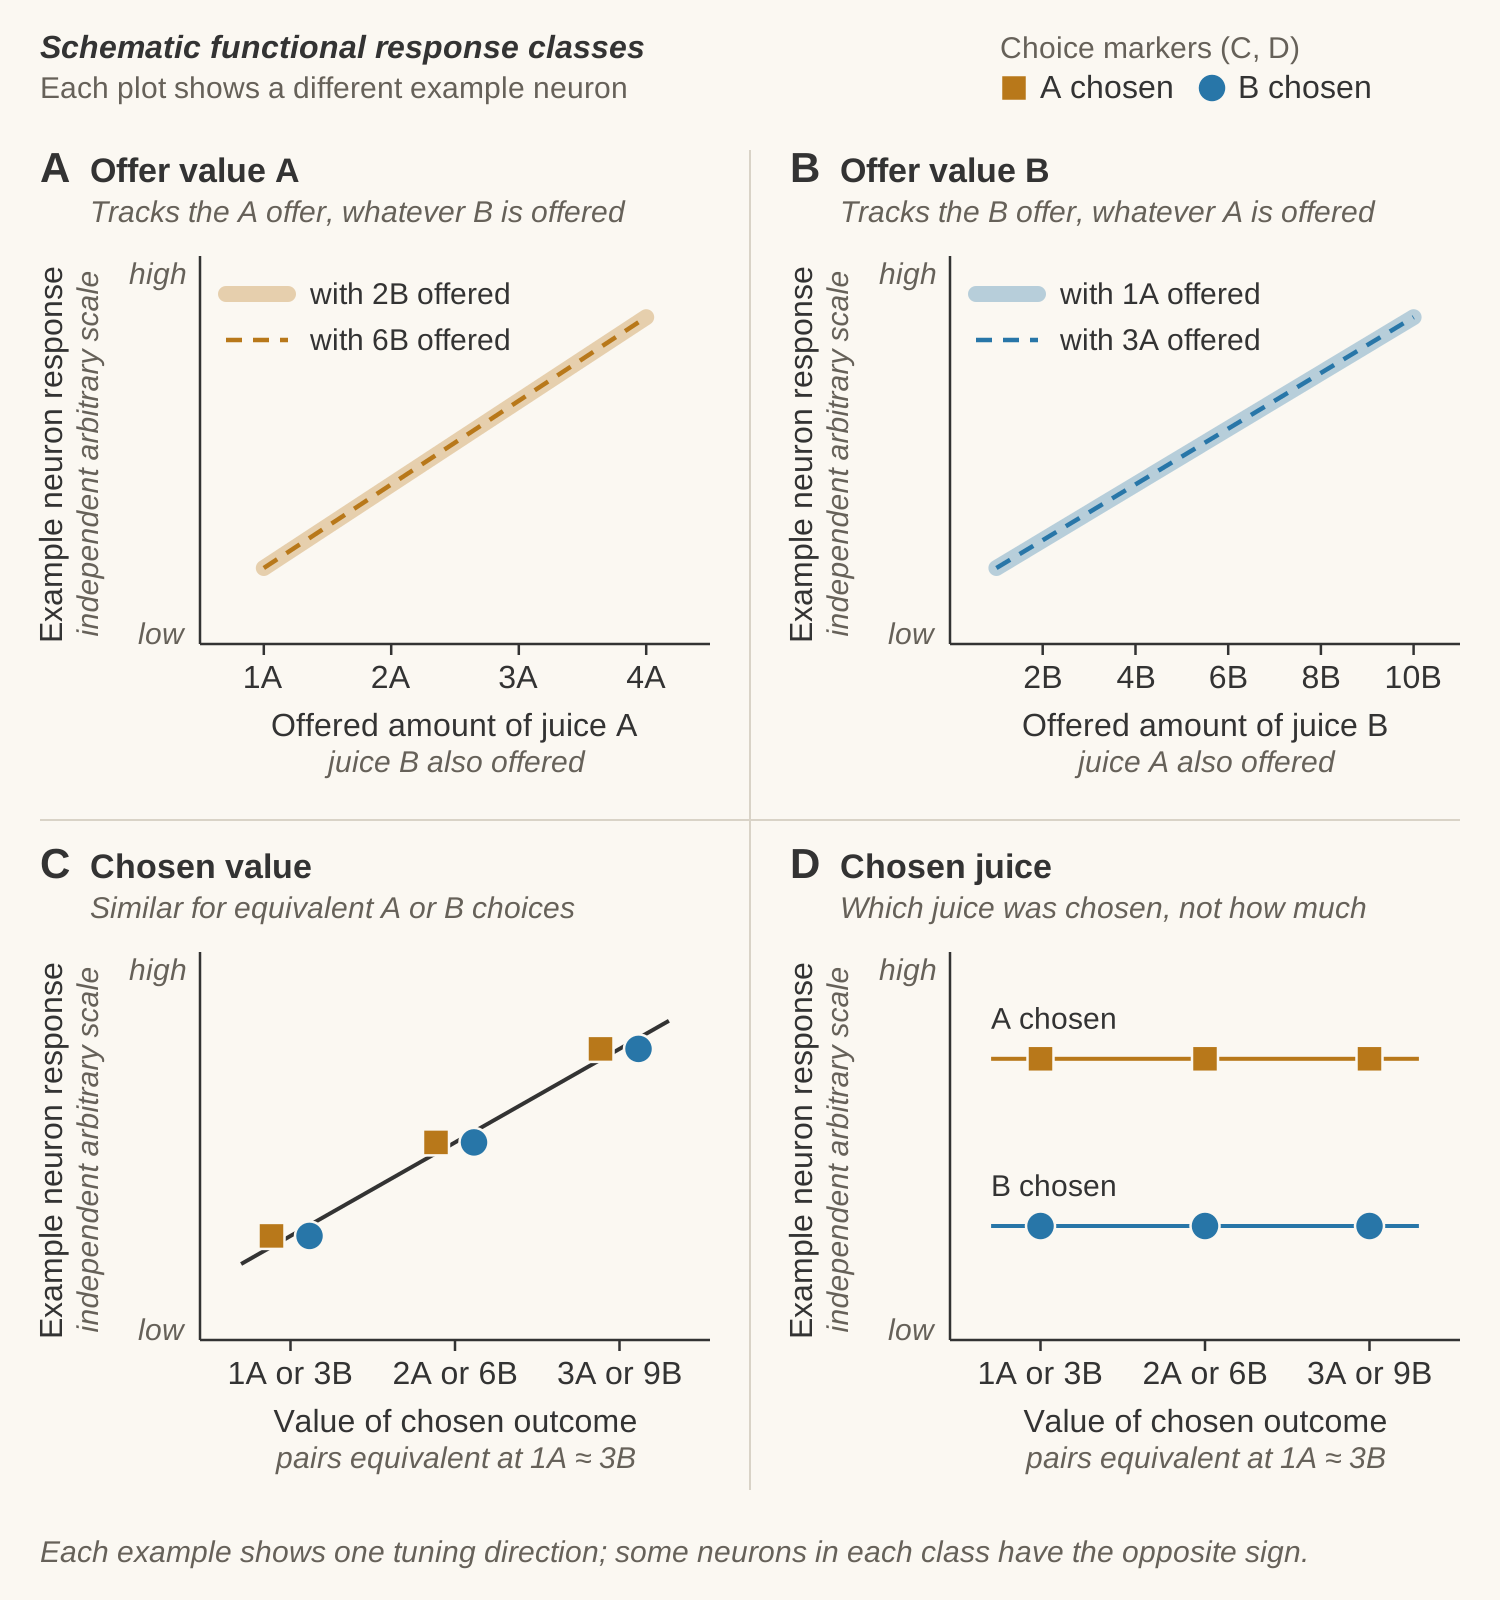
The exchange rate belonged to that animal under those conditions. It was inferred from repeated choices, and another animal could reveal a different preference. With this behavioral scale in hand, the investigators could ask what the neurons represented. Recordings in orbitofrontal cortex, on the ventral frontal surface described in Section 36.3, identified three prominent response types. Offer-value cells responded to the amount and value of one particular offered juice. Chosen-value cells tracked the value of the selected offer across the two juice identities. Chosen-juice cells distinguished which juice was selected; the original paper called this response taste.
The distinction among the cell classes is the central result. An offer-value cell associated with juice A was specific to that good; it was not a universal meter that responded identically to an equivalent offer of juice B. Chosen-value activity provided the more general signal, while other activity preserved the identity of the selected outcome. Nor should equal firing rates in two different neurons be assumed to mean equal value: individual neurons have their own response ranges and sensitivities. The evidence for a common format comes from how activity relates to behavior across conditions, particularly when a neuron’s relationship to chosen value generalizes across goods.
The locations of the offers varied, separating their identities and values from the direction of the saccade used to report the choice. This showed that the principal OFC signals were organized around the goods rather than simply around a leftward or rightward movement. It did not require a serial sequence in which all valuation finished before motor systems became involved. A coding distinction and a processing stage are different claims.
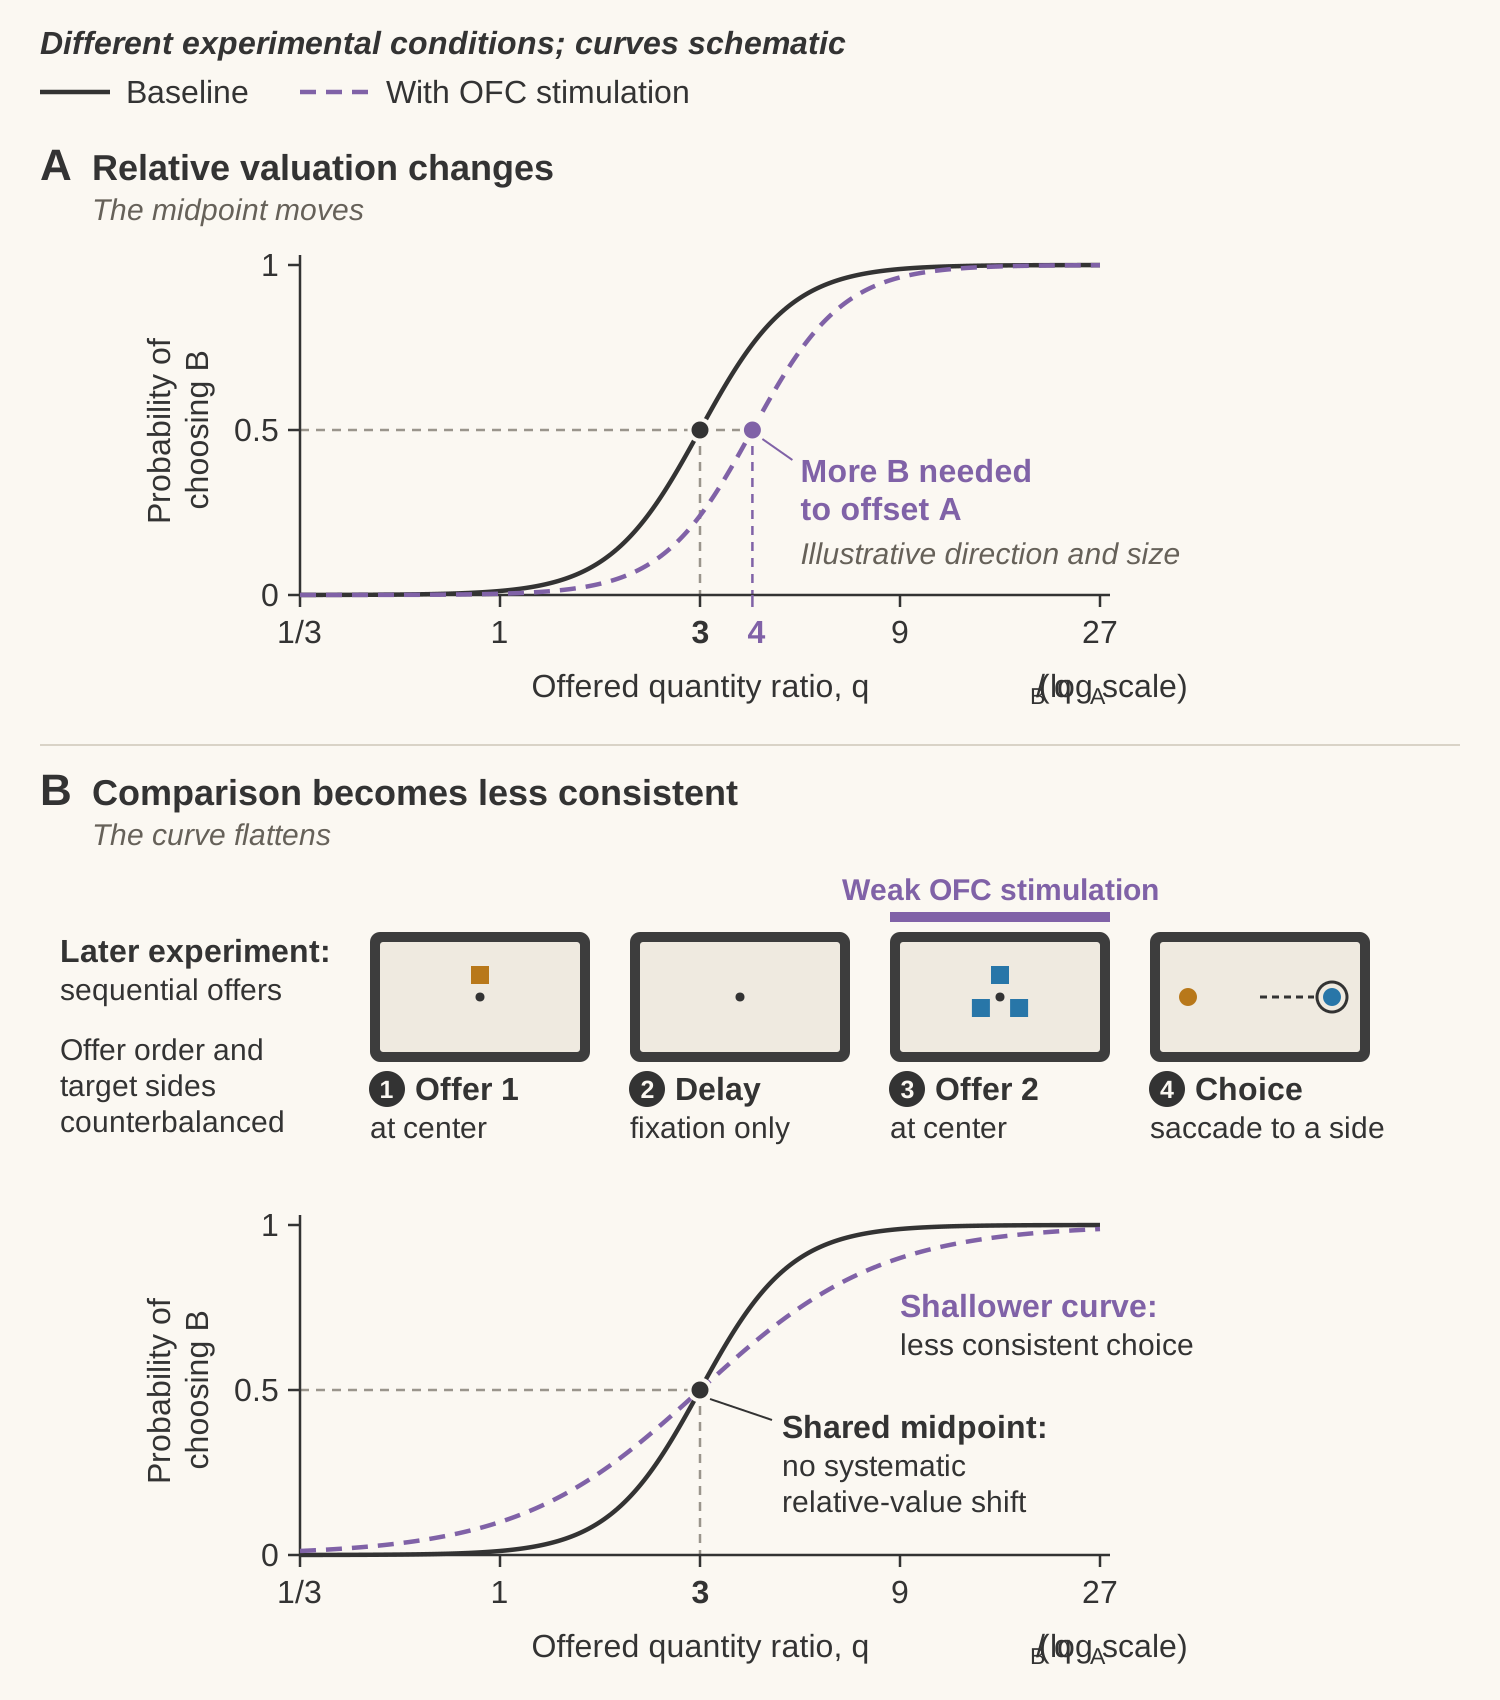
Subsequent perturbation experiments asked whether these signals participate causally in choice. Low-current electrical stimulation altered the values inferred from the monkeys’ decisions and biased choices in the predicted direction; stronger stimulation disrupted valuation and comparison and made choices more variable [@ballestaetal2020causal]. In a later experiment with sequential offers, weak stimulation delivered while the second offer was available increased choice variability without systematically shifting the estimated relative value of the juices [@ballestaetal2022comparison]. The latter result is especially informative: comparison became less reliable even though the behavioral exchange rate remained similar.
A psychometric choice curve makes the distinction visible. Changing relative value shifts the midpoint at which the two offers are equally likely to be selected. Increasing variability makes the curve shallower: the animal chooses less consistently around a similar midpoint. Together, the recording and perturbation experiments support a substantial causal claim. In this task, OFC populations represent the values and identities of offered goods and contribute to the comparison that produces a choice. The evolving activity of those populations is part of the mechanism through which one alternative gains influence over action.
37.4 Shared and specific value codes in humans
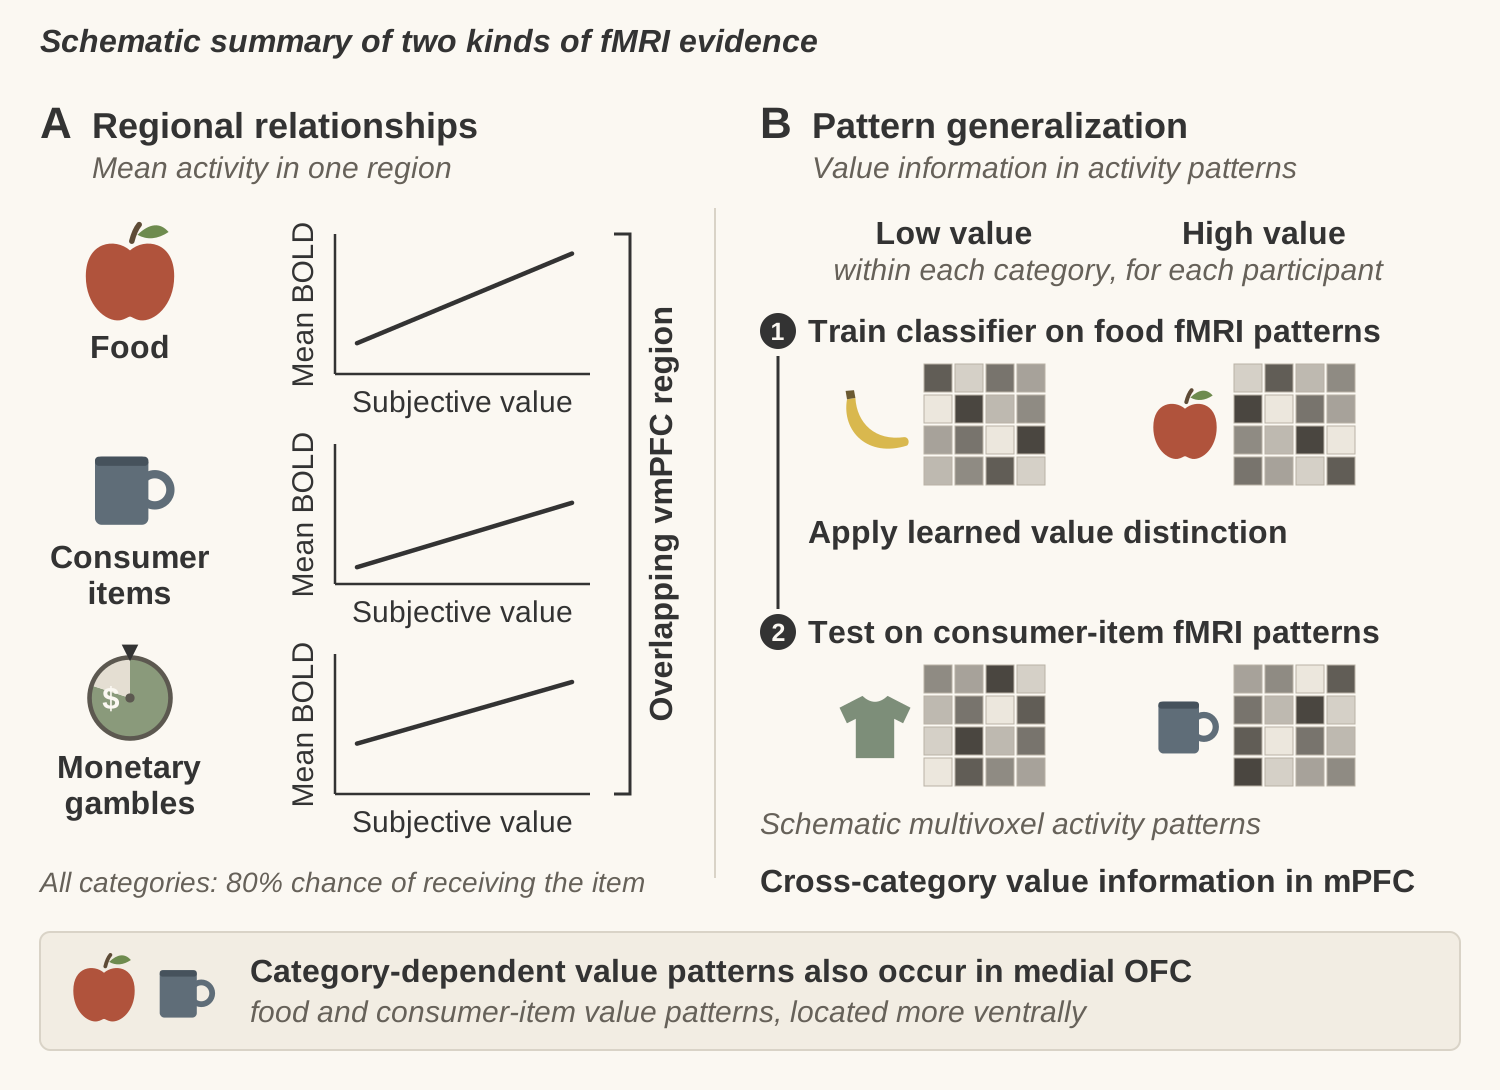
Human imaging extends the comparison to outcomes that differ more substantially than two juices. Chib and colleagues studied real purchasing decisions involving food, nonfood consumer items, and monetary gambles. Activity in an overlapping region of ventromedial prefrontal cortex covaried with participants’ valuations across all three categories [@chib2009common]. Money makes the comparison particularly useful. It has no fixed taste or consummatory response; its value depends on the possibilities for which it can be exchanged. The common signal therefore reaches beyond shared sensory properties.
The anatomical distinction needs the qualification made in the overview. The labels vmPFC and OFC overlap along the medial orbital surface, and their boundaries vary across studies. Differences between reported signals must therefore be read against the territories sampled, rather than assigned to two wholly separate cortical compartments.
A coordinate-based meta-analysis of 206 fMRI studies found recurring positive relationships between modeled subjective value and BOLD activity, especially in vmPFC and anterior ventral striatum. The pattern appeared during choice and outcome receipt and with both primary and monetary outcomes [@bartraetal2013valuation]. Regional convergence is meaningful, but the spatial scale matters. Overlapping BOLD responses do not establish that exactly the same neurons represent every good, and a value-related change in BOLD does not provide a universal linear readout of worth.
Pattern-based analyses can test distinctions that regional overlap leaves unresolved. McNamee and colleagues found category-independent value information in medial prefrontal cortex together with category-dependent patterns in more ventral medial orbitofrontal regions [@mcnameeetal2013category]. Howard and colleagues varied the identity and value of predicted food odors: OFC patterns carried identity-specific value information, whereas vmPFC carried a more identity-general signal [@howardetal2015identity]. In macaques, large-scale recordings also revealed different emphases within frontal circuits. OFC populations represented outcome flavor especially strongly, while ventrolateral prefrontal populations emphasized outcome probability; preference influenced both [@stollrudebeck2024preferences].
The resulting picture is richer than a single neural price. General and outcome-specific value signals coexist. Some activity supports comparison across different kinds of consequence. Other activity retains the identity, probability, and contextual information needed to predict those consequences and revise their significance. The findings fit the requirements of a controller that must choose now while remaining able to change its choice later.
The ventral striatum belongs inside this account. Its learned values, prediction errors, motivational signals, and action-related activity interact with cortical representations of expected outcomes and current state. Frontal activity participates in this recurrent competition; its own evolving state depends on striatal, thalamic, and other connected activity (Section 36.5). The question is how these interactions make particular consequences effective in choice.
37.5 The body changes the value of the expected outcome
Comparison is useful only if the values being compared remain appropriate to the organism. A change in bodily state provides a particularly clear test, because it can change the significance of an outcome while leaving the outcome itself intact.
37.5.1 Selective satiety preserves the identity of what was eaten
Eating one food to satiety usually reduces the desire for that food more than for other foods. The selectivity matters. A general reduction in reward responsiveness would not explain why a different food remains attractive.
In monkeys, OFC neurons responding to the odor or sight of a food reduced their responses after the animal ate that food to satiety. Responses to other foods were relatively preserved [@critchleyrolls1996satiety]. The image and odor had not changed; the organism’s relation to the predicted food had. A human conditioning experiment extended this result to learned cues. Participants first learned that two arbitrary visual cues predicted different food odors, then consumed one associated food to satiety. When the cues were presented again without the odors, OFC and amygdala responses declined selectively for the cue predicting the devalued outcome [@gottfriedetal2003devaluation]. The change concerned something expected, rather than a taste presently in the mouth.
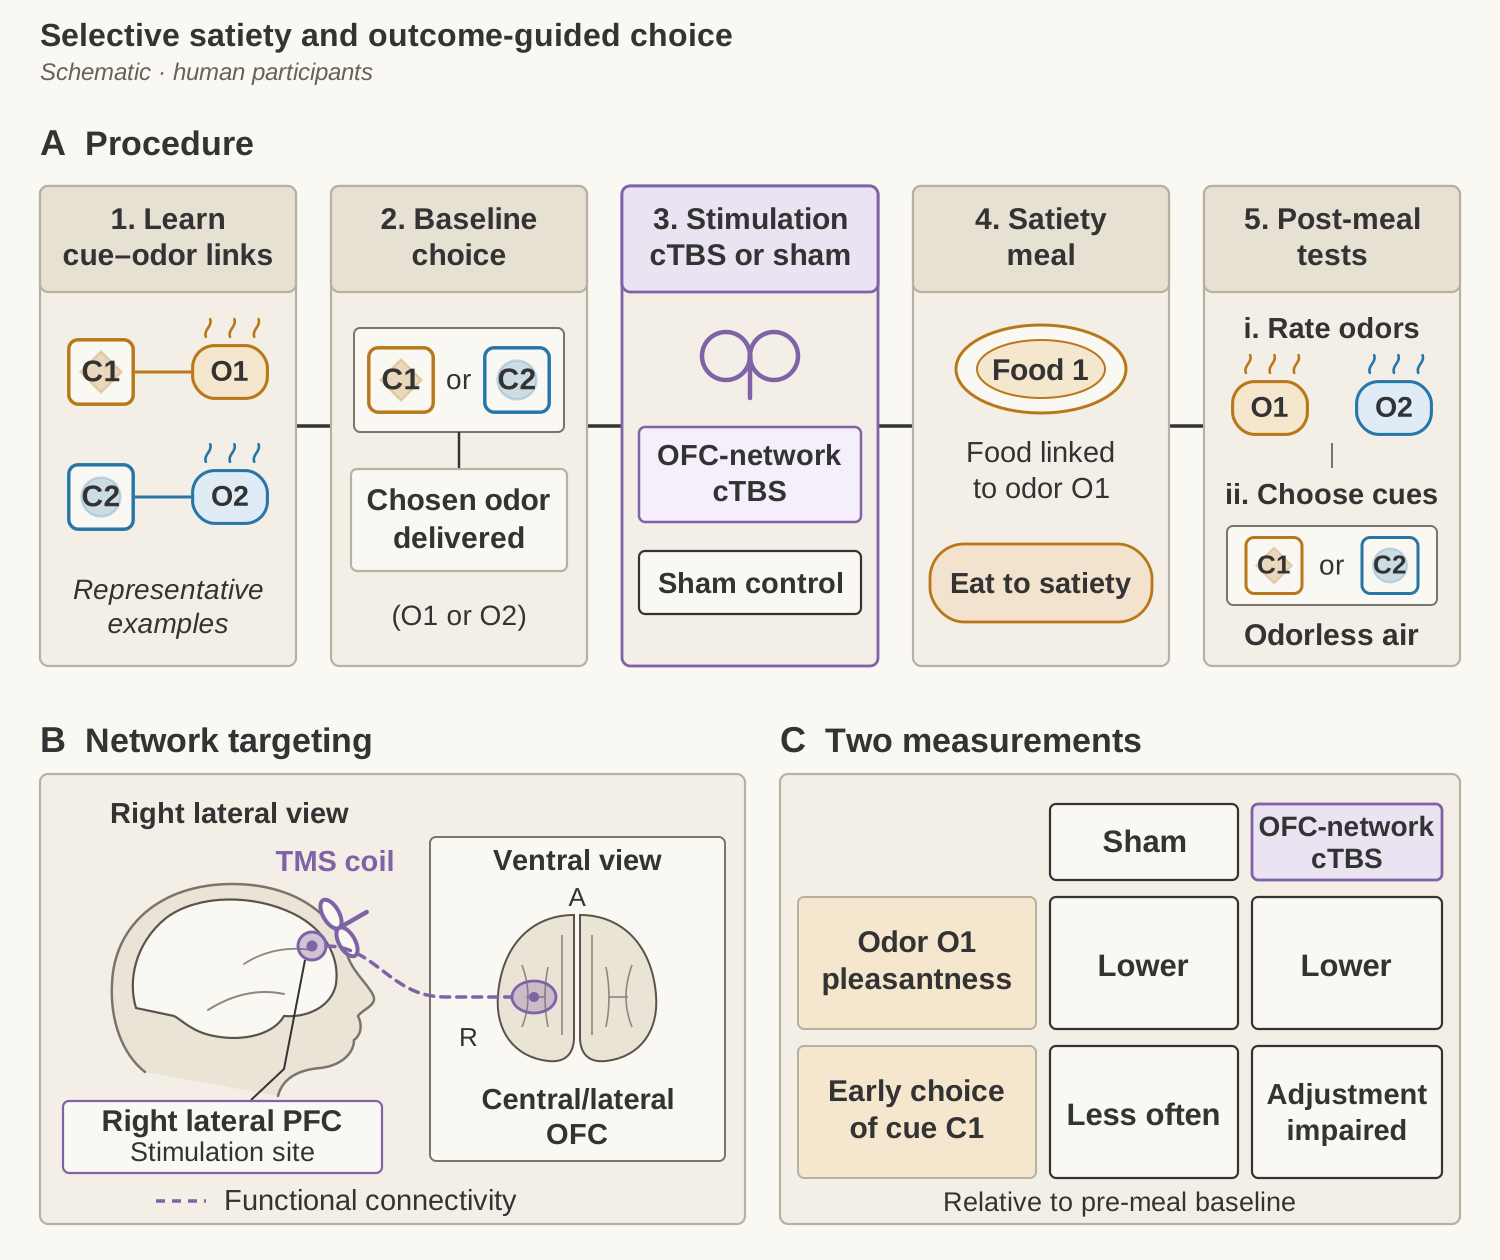
Howard and colleagues tested the causal contribution of this network with theta-burst stimulation. Because orbital cortex is difficult to reach directly with conventional TMS, they stimulated a lateral prefrontal site selected for its connectivity with OFC before the satiety meal. After this perturbation, participants still rated the sated food odor as less pleasant, but their initial choices among visual cues failed to adjust normally to that devaluation [@howardetal2020stimulation]. The distinction is revealing. The outcome had lost its appeal; the altered network did not use that change effectively when the outcome was represented by a predictive cue.
Selective devaluation therefore requires several relations to remain available together: this cue predicts this food, the food has just been consumed, and its desirability has declined while another food remains attractive. Identity and value must be separable enough for the value to change without losing the prediction that makes the change relevant.
37.5.2 A new need can change an old prediction
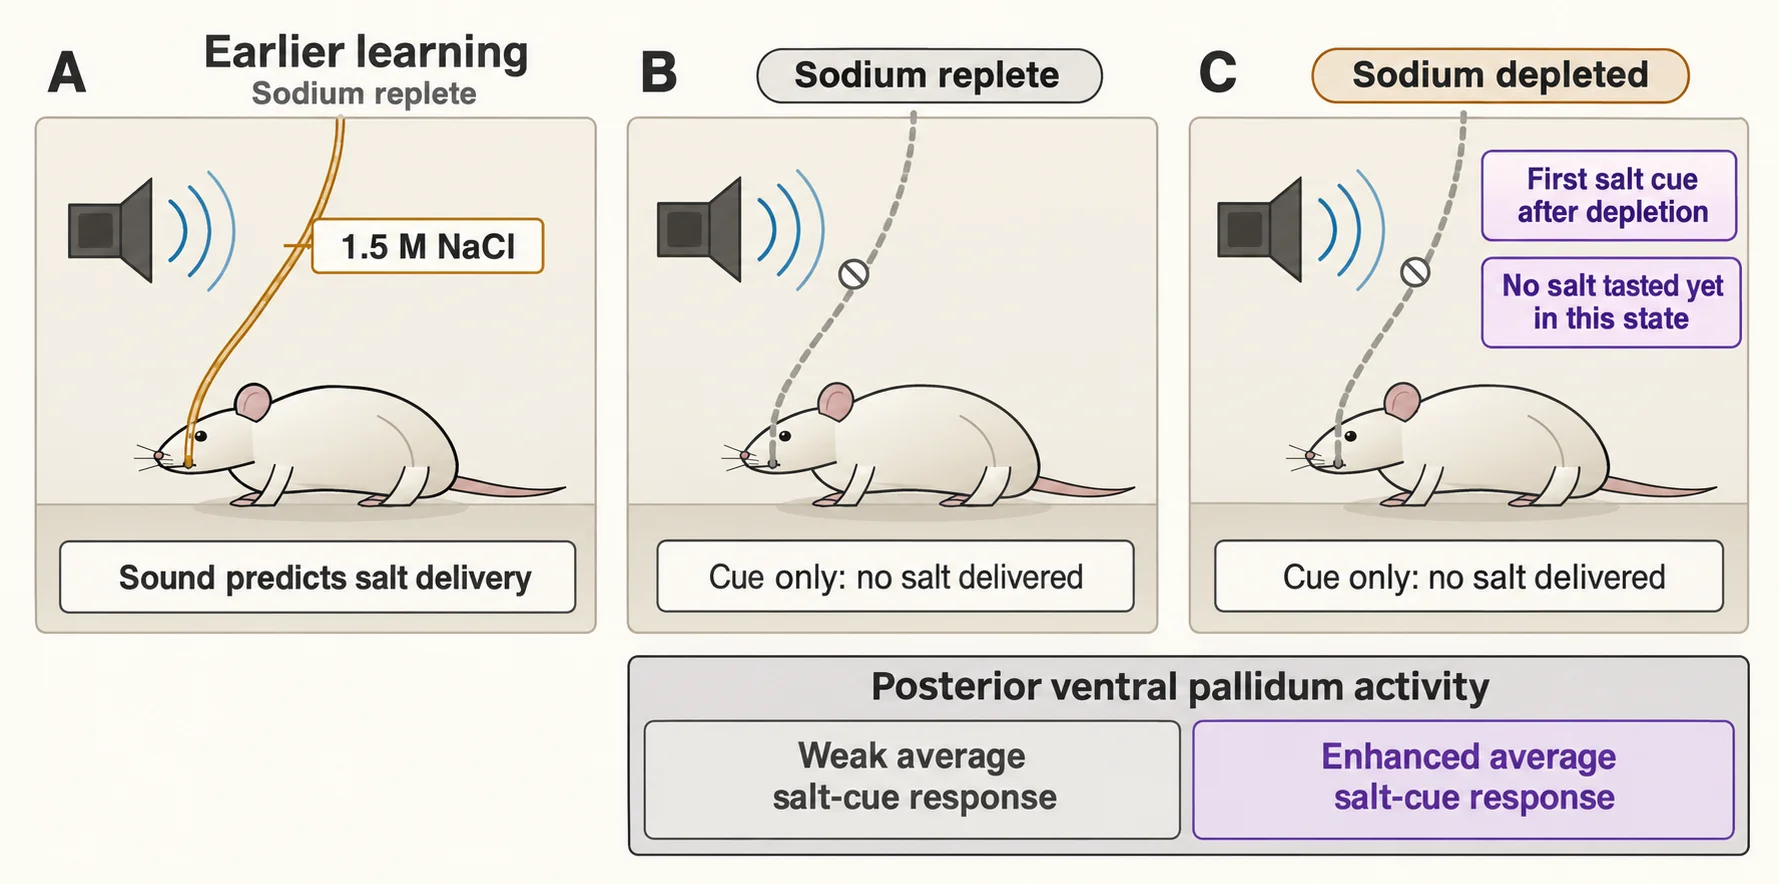
Physiological state can also increase the motivational force of a cue before the animal experiences the outcome in its new condition. In the sodium-appetite experiment introduced in Chapter 35, rats learned a cue predicting a highly concentrated salt solution that was normally unpleasant. Sodium depletion later transformed their response to that cue. On its first presentation in the depleted state, before the rats had tasted the salt under those conditions, average cue-evoked firing among responsive posterior ventral pallidum neurons increased [@tindelletal2009dynamic].
The new response could not have been learned from a newly rewarding salt taste, because that experience had not yet occurred. A previously learned prediction interacted with the current physiological state. The result limits an account in which the cue merely retrieves an unchanged value acquired during earlier experience. It supports a more flexible mechanism in which need can alter the motivational significance of what the cue predicts. The experiment concerns that revaluation; it does not, by itself, identify every computation or representation responsible for it.
37.5.3 Anticipation changes regulation before the deficit develops
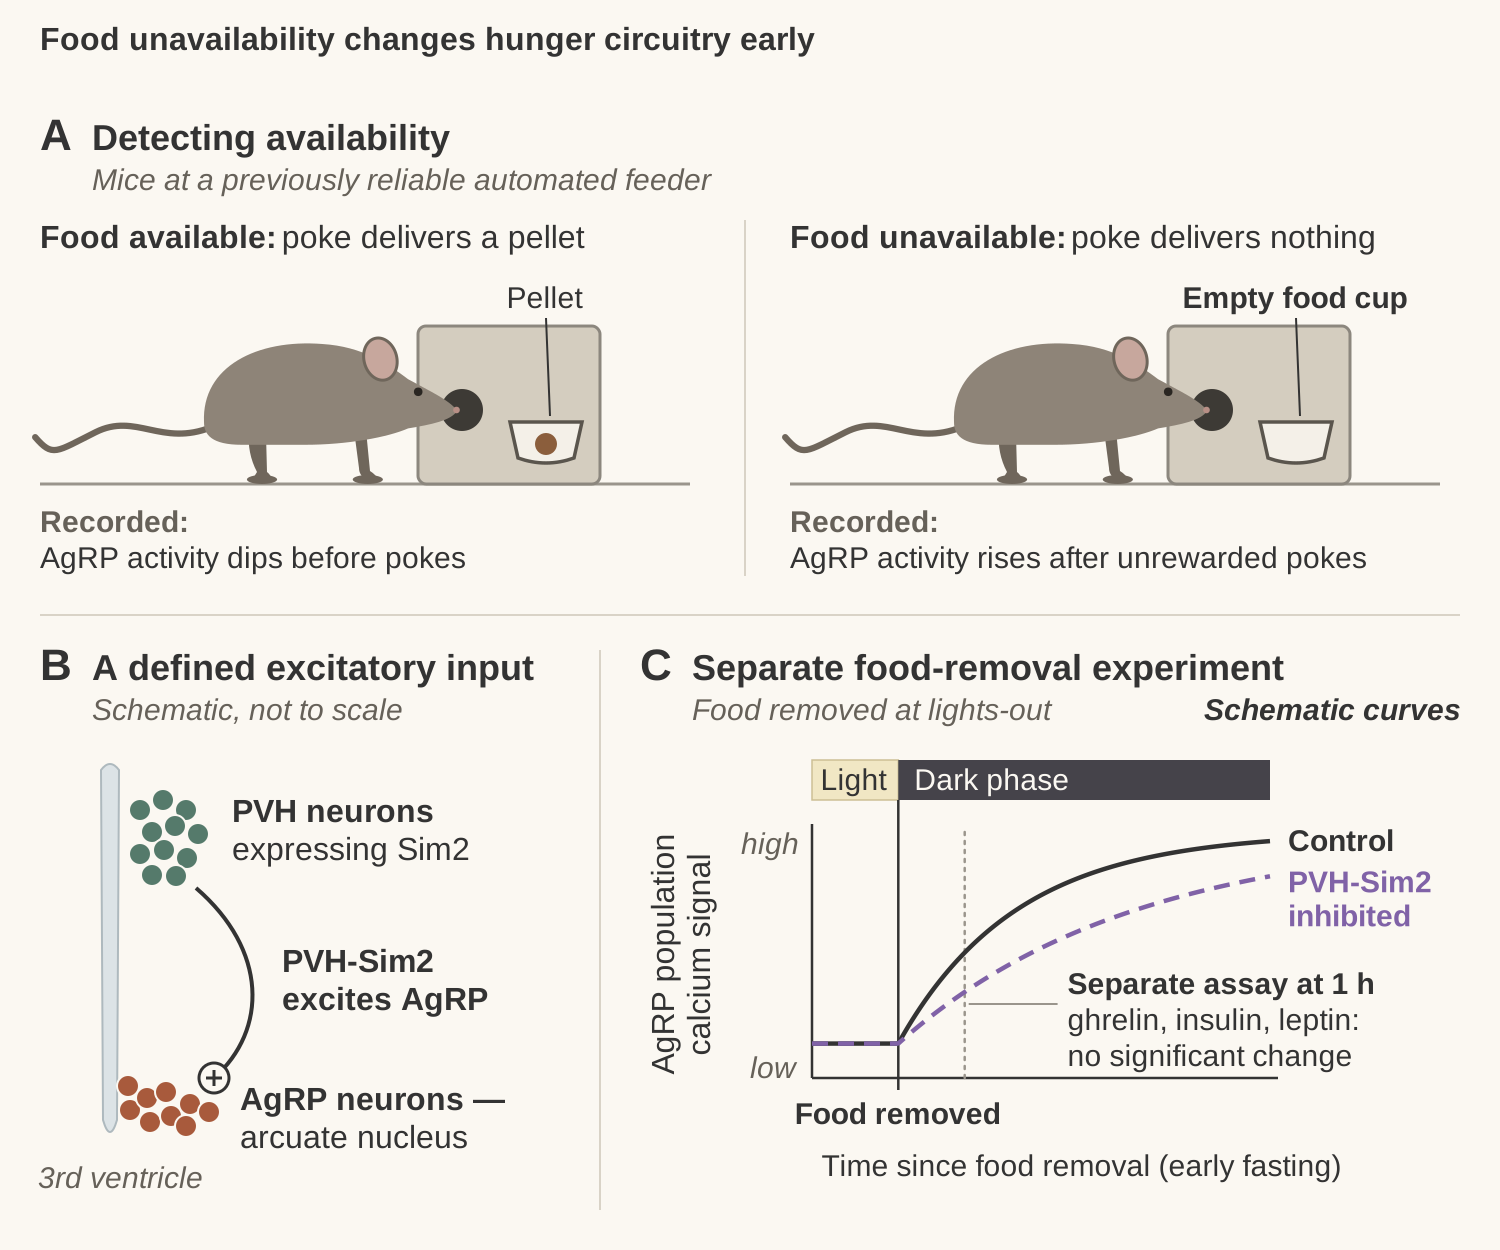
Predictive regulation can act earlier still. Food-related cues rapidly inhibit hunger-related AgRP neurons before nutrients have reached the circulation. Experiments on hunger and thirst circuits also show that activity in these systems can carry aversive motivational significance, linking need to the learned value of its relief [@betleyetal2015need]. A predicted consequence can therefore change the regulatory system before the body has obtained it.
Walker and colleagues demonstrated a complementary effect in mice: removing food at the start of the active period produced an early rise in AgRP activity. Excitatory input from paraventricular hypothalamic neurons expressing Sim2 contributed to this response; inhibiting those neurons slowed the rise [@walkeretal2026anticipating]. The findings support an anticipatory contribution to allostasis: information about food availability can influence feeding regulation in anticipation of the energy deficit that continued fasting would produce.
These findings also keep the frontal argument in proportion. Anticipation is already present in hypothalamic circuitry. Frontal elaboration extends the range of circumstances that can influence behavior, drawing on remembered contexts, inferred transitions, alternative courses, and socially learned goals. It operates within a body whose regulatory systems are themselves predictive.
The ecological implication can be illustrated by a route toward water. The water may deserve little effort immediately after drinking but become worth seeking before a long crossing through heat. Its anticipatory value depends on both the consequence of the action and the state expected when that consequence becomes available. Similarly, shade can be sought before overheating, and shelter before an expected danger arrives. These examples express the chapter’s control interpretation: an outcome can matter because it preserves the organism’s capacity to remain within viable conditions later.
37.6 Value belongs to an outcome in a situation
The state conditioning value also includes the situation outside the body. A visible cue can predict different consequences in different contexts, and the relevant context may itself be hidden. Recent history, location, a task rule, or an unobserved transition can determine which situation applies. The animal must establish what the cue means here before its expected consequence can guide an appropriate response.
Schuck and colleagues used a human task in which the visible event did not supply all the information needed to identify the current task state. Relevant information had to be carried forward from previous events. Multivoxel patterns in OFC distinguished hidden states needed to organize performance [@schuck2016map]. This connects orbital activity to the representation of the situation within which outcomes acquire value. In the terms introduced in Section 36.1, such information contributes to a control state when it changes how the organism uses a cue or recruits an action.
Sensory preconditioning provides a complementary test in rats. Animals first learned a neutral relation in which cue A preceded cue B. Later, B was paired with food. At test, responding to A could draw on the previously learned relations, \(A \rightarrow B \rightarrow food\), although A had never been directly paired with food. Temporary OFC inactivation during testing abolished the elevated response to A while sparing the response to the directly reinforced B cue [@jonesetal2012inferred]. In this experiment, OFC was necessary for using the learned associative structure to guide behavior toward an indirectly predicted outcome. The result supports inference from that structure without requiring that the animal consciously traverse a chain of propositions.
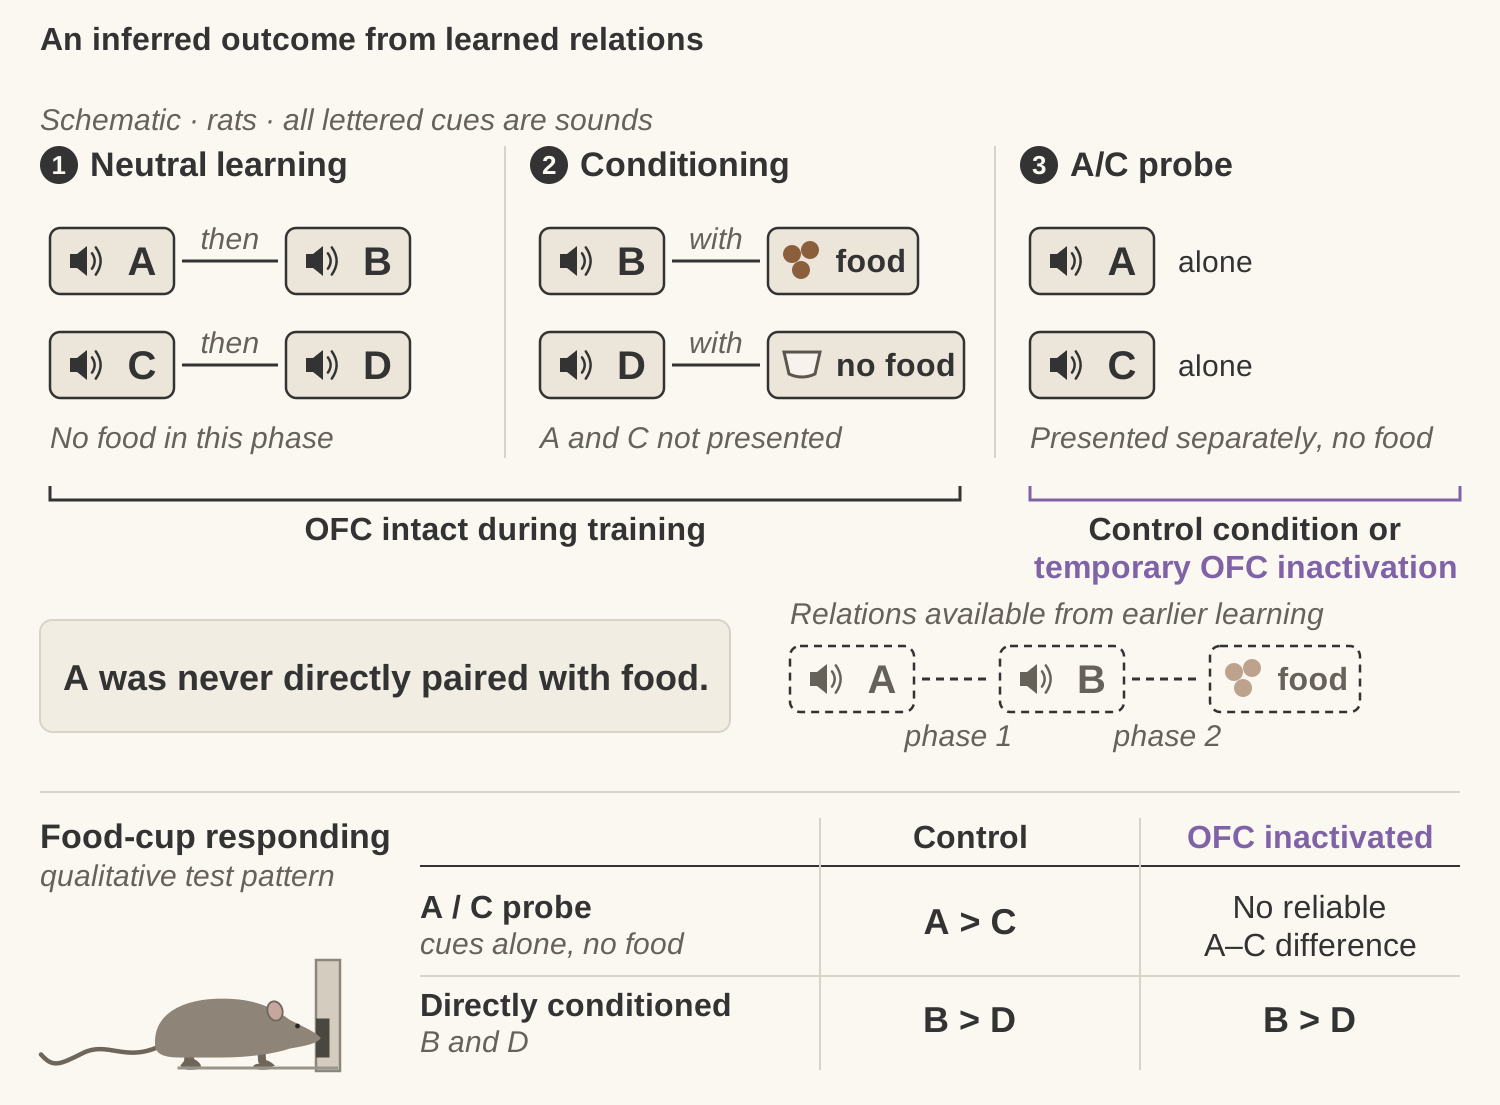
Several related experiments can now be distinguished. Devaluation changes an outcome’s desirability while preserving its identity. Reversal changes which outcome a cue predicts. Latent-state inference identifies a situation whose decisive features are absent from the current sensory input. Model-based inference uses learned relationships to derive an expectation that need not have been acquired through direct reinforcement of the tested cue. They share a demand for flexible use of prior learning, but the information that changes is different in each case.
I take these findings to support a broader view of orbital cortex: it helps make an expected outcome meaningful within a represented situation. That is a synthesis of the evidence, rather than a claim that one experiment has established a complete theory of OFC. The juice-choice studies demonstrate a causal contribution to valuation and comparison; the devaluation and inference studies reveal the importance of retaining the relations from which a current value can be derived. A satisfactory account has to explain both.
37.7 Choice as recurrent control
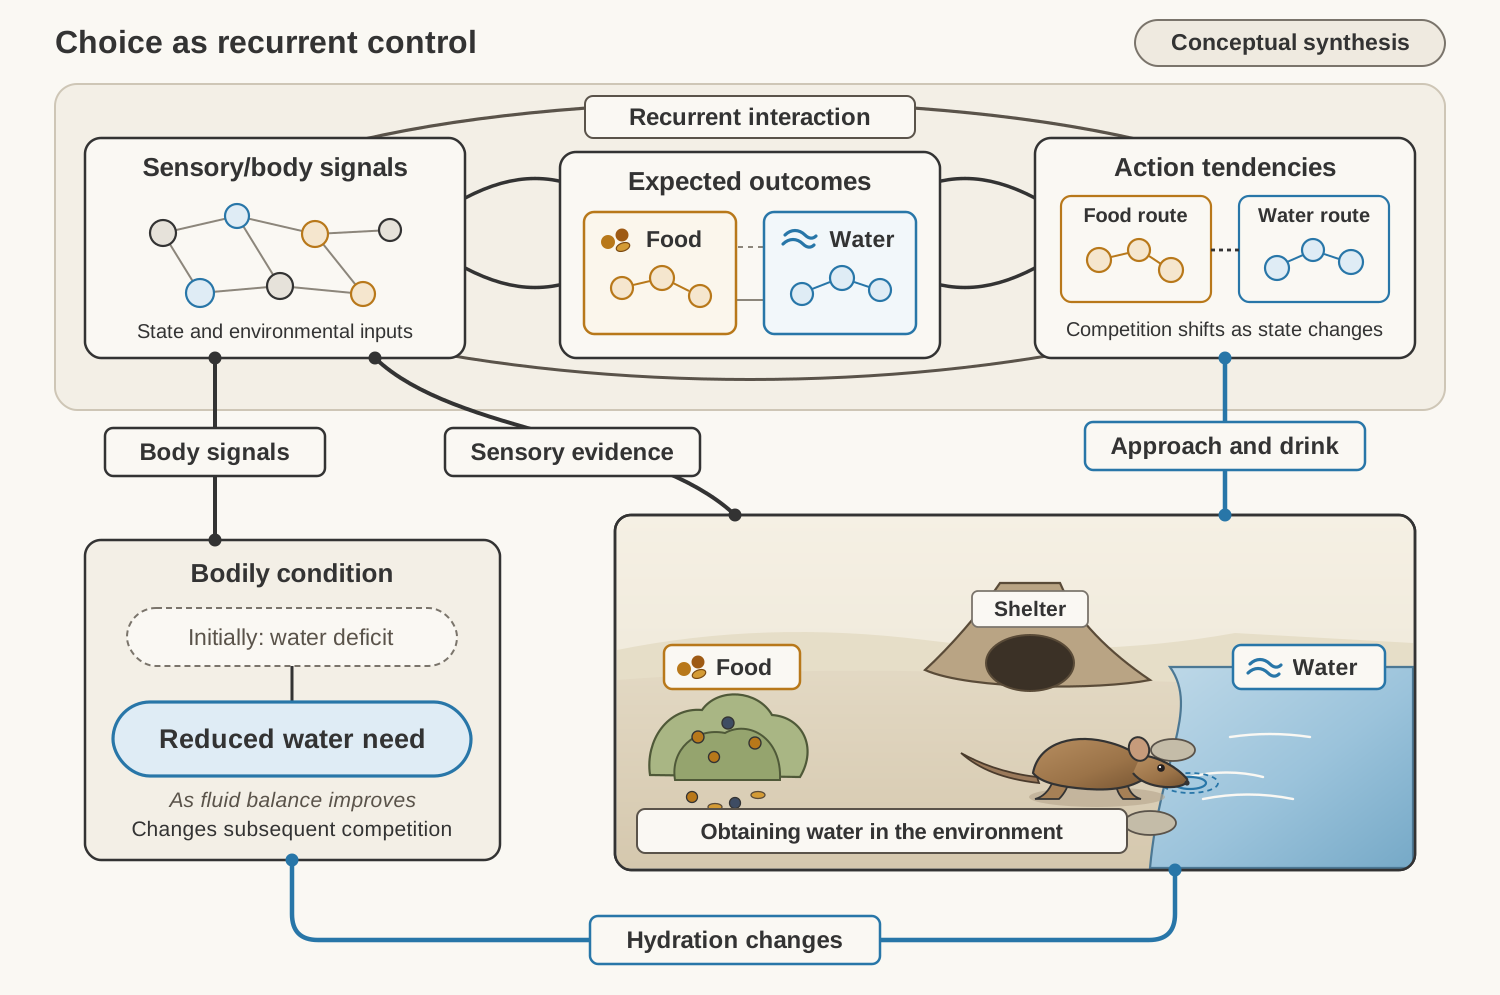
The physical requirements become clear when selective satiety is followed through the system. Eating changes bodily signals and the responses associated with a particular food. The food’s sensory identity and its learned relation to a cue remain available. When the cue appears again, it encounters a network whose current state differs from the state in which the original preference was learned. Its influence on choice changes accordingly. If another food remains attractive, the competition between the available actions can change even though neither cue has changed.
The experiments locate parts of this process. OFC and amygdala responses to food-predictive cues change selectively after devaluation; disrupting an OFC-connected network can impair the adjustment of cue-guided choice while preserving the decline in the food odor’s reported pleasantness [@gottfriedetal2003devaluation; @howardetal2020stimulation]. Representing an outcome, changing its value, and using that value to guide action are connected achievements that can be experimentally separated.
Their integration depends on the anatomy developed in the overview. Information about outcome identity reaches particular orbital networks through sensory and temporal association connections. Bodily condition and learned context enter through differentiated insular, amygdalar, hypothalamic, and memory-related routes (Section 36.4). Some pathways are direct; others act through intervening structures. The distinction matters: tracing a connection does not establish which need or prediction it carries during a choice.
Orbital and ventromedial cortex participate with striatum and thalamus in recurrent systems through which expected outcomes can influence action. Thalamic activity helps sustain and reshape cortical states, so these loops do more than transmit a finished choice (Section 36.5). Frontal activity can also influence cortical action systems through selected premotor and medial motor connections, and bodily preparation through selected hypothalamic and brainstem routes (Section 36.6). These concurrent routes provide several ways for a predicted consequence to alter the organism while returning sensory and bodily information changes the prediction.
The control account concerns how these interactions unfold. Current state changes which consequences matter; the expected consequences change attention and preparation; action changes the body and environment; the resulting evidence revises what is expected next. A decision variable is effective only through the connections by which it changes this ongoing activity. Describing a value signal identifies one useful feature of the process. Explaining choice requires the dynamics through which that signal and the other relevant information alter action.
The common-currency hypothesis retains a clear role within this account. General value signals can make dissimilar consequences comparable, while specific representations preserve the information needed to anticipate and revise them. The animal’s changing circumstances continually alter the terms of comparison.
37.8 Coda: a value must remain in control
Choosing a valued outcome begins a longer problem. The outcome may disappear from view while intermediate actions are completed. Another cue may offer an easier reward. The body may change enough to justify reconsidering the original choice. A controller must keep the selected consequence effective across distraction while remaining responsive to evidence that the choice is no longer appropriate.
That is the problem of Chapter 38. A consequence can matter when the offers are visible; the next question is how its influence survives as the organism moves through the world.
The evidence. Subjective value changes with bodily and task state. In monkey juice-choice experiments, OFC populations distinguish offer value, chosen value, and chosen identity, and stimulation alters valuation or comparison. Human imaging identifies recurring value relationships in vmPFC and anterior ventral striatum, alongside more outcome-specific representations. Selective satiety, sodium need, and inferred task relations can change responses to predicted outcomes. OFC perturbations reveal a causal contribution to several forms of flexible outcome-guided behavior.
The interpretation developed here. Valuation is part of an embodied controller. Common decision variables coexist with representations of outcome identity and situation, allowing comparison to remain responsive to present and anticipated conditions. The recurrent account joins these component findings into an explanation of how consequences gain and lose influence over action.
The open questions. The evidence does not establish one universal currency for every kind of choice. The cellular organization of general and identity-specific signals in humans remains unresolved, as does the balance between goods-based and action-based representations across tasks. A fuller account must explain how state, attention, learned relationships, and neural population dynamics change the causal contribution of each circuit as a decision develops.