38 Holding the Line
Maintained Control Without a Working-Memory Module
38.1 A future must survive its cue
Chapter 37 ended with a problem that valuation alone cannot solve. An expected outcome can gain control of action and then disappear from view. The animal must cross a changing environment before the outcome is reached, and the body in relation to which that outcome was valued continues to change along the way. The loop in Figure 37.10 therefore continues throughout the journey, not only when a new choice is offered.
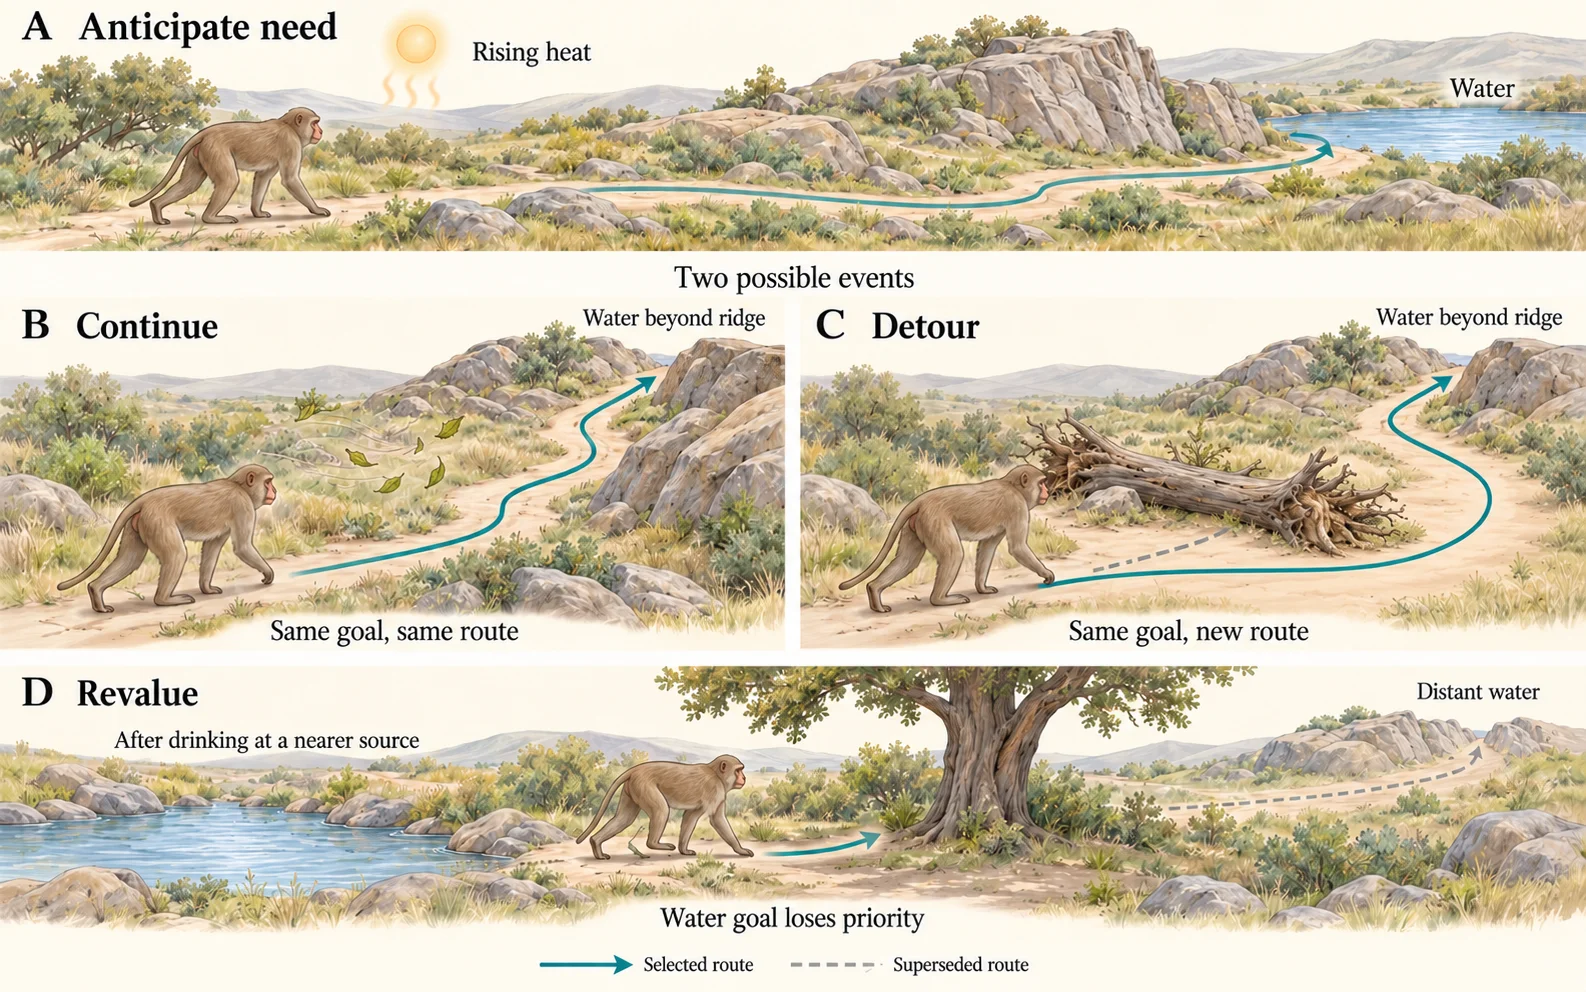
Consider an animal that leaves a feeding area for a distant source of water before dehydration becomes severe. The action is allostatic: present behavior is organized around a predicted future state. Once the route has begun, the water may no longer be visible. Intermediate movements must be completed, landmarks must be used, and immediately available food or novel movement may compete for orientation. The expected water must continue to influence behavior although neither the water nor a severe fluid deficit is currently present.
Persistence alone would be maladaptive. A predator may enter the route. Cooling rain may reduce the expected heat load. A nearer source of water may appear, or the remembered path may prove blocked. The controller must reject events that do not change the problem while incorporating events that do. It must remain stable against distraction and flexible in response to evidence.
Adaptive control requires selective persistence: a future must remain effective after its cue disappears, but it must lose control when it no longer justifies the action.
The anatomical framework is already in place. Section 36.3 distinguished lateral frontal association territories from their orbital, medial, and motor neighbors; Section 36.5 placed them within cortical, thalamic, and basal-ganglia interactions. This chapter asks how activity within that architecture keeps a condition effective across time. The psychological literature usually places much of this behavior under working memory. That term remains useful, but it must not be mistaken for the name of a neural organ or a single physiological mechanism.
38.2 Working memory is a psychological construct
The phrase working memory belongs first to psychology. It names a family of behavioral capacities involving the temporary availability and use of information. Information that is no longer supplied by the current stimulus can support comparison, rule use, calculation, comprehension, or action. People differ reliably in performance on tasks designed to measure that availability, and the construct can organize useful predictions at the psychological level.
None of this requires a one-to-one neural counterpart. Delayed saccades, digit span, mental arithmetic, sentence comprehension, the n-back task, and following a briefly stated rule are all called working-memory tasks. They differ in what must be represented, what transformation must be performed, what response is prepared, how interference is introduced, and whether any item must remain in the focus of attention. A term that groups these behavioral demands does not thereby identify one neural buffer shared by all of them.
The error is subtle because the grammar encourages it. Once working memory becomes a noun, it is easy to ask where the brain stores it, how large its capacity is, or which region serves as its executive. These are legitimate questions when the operations and measurements are specified. The error is to assume that the shared task label guarantees a shared neural object. Activation in a working-memory task can then be interpreted as activation of working memory itself, before the experiment has distinguished retention from attention, preparation, or response selection.
The appropriate analysis moves in the other direction. A task should be decomposed into operations and variables that nervous tissue can implement. What information is absent from current input? Which sensory or mnemonic representation must remain consequential? Is the subject monitoring a location, retaining an identity, expecting an event, applying a rule, preparing a movement, estimating elapsed time, or protecting one representation from interference? Which parts of the task require sustained activity, altered synaptic efficacy, recurrent interaction, or a change in the gain applied to later input?
A psychological construct can be valid without being a neural module. The neural explanation begins when the task is decomposed rather than when the construct is assigned to cortex.
This distinction does not make the physiological evidence disappear. It makes that evidence more important. Lateral frontal activity recurs across many tasks in which information, attention, expectation, or preparation must remain effective over time. The convergence appears in monkey single units, human lesion studies, slow cortical potentials, and functional imaging. The central empirical fact is robust. Its interpretation is broader than a dedicated store called working memory.
At the psychological level, working memory summarizes regularities in behavior: recent information can remain available, capacity is limited, interference matters, and temporary availability predicts performance in many tasks. Those are legitimate phenomena.
At the neural level, the same tasks recruit different combinations of sensory cortex, parietal cortex, hippocampal and medial-temporal systems, frontal cortex, thalamus, basal ganglia, and motor systems. The mapping is many-to-many. A delayed-response task does not isolate a mental substance called working memory, and a region activated by that task does not become its anatomical home.
The useful bridge between levels is an explicit account of the task. Psychological constructs describe organized behavior. Neural mechanisms explain how particular variables remain available, selected, transformed, and connected to action in particular circumstances.
38.3 The delay period made an absent variable visible
The strongest physiological evidence begins before the term working memory became dominant. In 1971, Joaquín Fuster and Garrett Alexander recorded neurons in monkey prefrontal cortex and the mediodorsal thalamus during a delayed-response task. Many neurons changed their firing when the cue appeared, and some remained above their intertrial firing rate throughout the delay [@fusteralexander1971delay]. Activity in frontal and thalamic neurons therefore bridged the interval between information and action. The earliest observation already drew attention to a frontothalamic system. Recording activity in both structures did not, by itself, establish that reciprocal interaction sustained the activity; the causal tests came later.
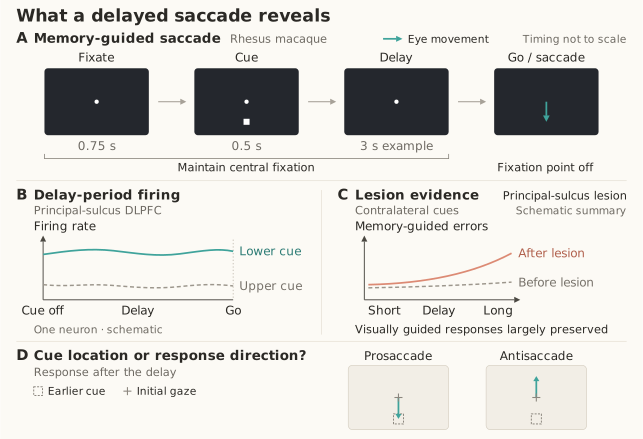
Funahashi, Bruce, and Goldman-Rakic later made the represented variable much more precise. In the oculomotor delayed-response task, a monkey fixated a central point while a peripheral target appeared briefly. The target disappeared, fixation continued through a blank delay, and the disappearance of the fixation point instructed a saccade to the remembered location. Retinal stimulation and eye position were controlled during the delay, and the direction and timing of the eventual response could be measured exactly [@funahashi1989mnemonic].
Neurons around the principal sulcus in macaque dorsolateral PFC showed spatially selective delay activity. This is the lateral association territory introduced in Section 36.3, not primary motor cortex or the frontal eye field. One neuron might remain active after a cue in the upper-left visual field but not after an otherwise identical cue in the lower-right field. The preferred region was called a memory field. Across the population, the pattern of activity contained information about a location that the retina no longer supplied.
A complementary lesion experiment tested the contribution of the tissue. Lesions in and around the principal sulcus produced delay-dependent errors for remembered locations in the contralateral visual field while leaving visually guided saccades substantially intact. Errors increased as the blank interval lengthened [@funahashietal1993lesions]. The relevant frontal tissue was therefore necessary for normal performance under these task conditions. A lesion disrupts local processing and its network interactions; it does not selectively remove delay-period firing. The result supports a causal contribution of the region without identifying sustained firing as its only necessary mechanism.
These experiments established a firm result: prefrontal population activity can preserve task-specific information after the eliciting stimulus has disappeared, and disruption of the relevant tissue impairs the behavior that depends on that information. They did not establish that working memory, as a psychological faculty, had been found inside the principal sulcus.
The task itself contains more than retrospective memory. The cued location can also be a focus of attention and is the target of a future saccade. The standard task does not separate those variables. Later antisaccade experiments separated the remembered cue location from the required movement direction. Most of the studied neurons followed the cue location; a smaller group followed the forthcoming saccade direction [@funahashietal1993antisaccade]. The distinction matters: a representation of where the cue had appeared could help prescribe a movement toward it or support a movement away from it. Retaining a location and specifying a response are separable operations.
Persistent firing should therefore be described without either minimizing or personifying it. It is not a neuron “holding an image in mind.” It is sustained, selective activity through which an absent variable continues to alter the state of a circuit and the probability of a later action.
38.4 The frontal regularity is broader than memory
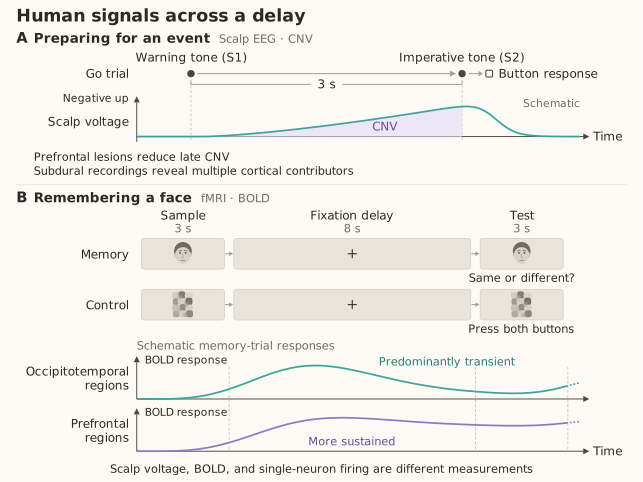
A second experimental tradition reached the same general problem without asking subjects to retain a visual item. Walter and colleagues presented a warning stimulus followed, after a predictable interval, by an imperative stimulus that required a response. A slow negative voltage developed over the scalp during the interval. They called it the contingent negative variation, or CNV, and described it as an electrical sign of association and expectancy [@walteretal1964cnv].
The CNV occurs while the organism is waiting in a task-defined state. The warning signal has changed what the next event means, when it is expected, and which response may be required. Anticipatory attention, temporal expectancy, motivation, and motor preparation all contribute. There need be no vanished object stored in a buffer. What persists is a relation among the warning cue, the expected event, the task rule, and the prepared response.
Lesion and intracranial evidence place frontal cortex within this sustained preparation without assigning the potential to one source. Patients with prefrontal lesions showed a marked reduction of the late CNV [@rosahlknight1995cnv]. Subdural recordings revealed CNV activity at multiple cortical sites, including prefrontal, supplementary sensorimotor, primary sensorimotor, temporal, and occipital regions [@hamanoetal1997cnv]. The scalp waveform reflects the summed contribution of distributed electrical generators. These results support frontal participation in sustained preparation; the waveform alone does not identify which rule, stimulus, or action is represented.
Functional imaging supplied a third scale of observation. In a delayed face task, Courtney and colleagues separated transient responses to visual events from activity sustained across the blank interval. The relative contributions differed: three occipitotemporal regions responded predominantly to the visual events, while three prefrontal regions showed more sustained responses across the delay [@courtneyetal1997sustained]. The result supports a distinction within the distributed system, not a claim that every participating region carries the same sustained signal. BOLD activity also cannot establish that individual neurons fire continuously.
The convergence across methods should not be explained away. Single neurons, field potentials, lesions, and BOLD measurements all implicate frontal systems in temporally extended task organization. The shared involvement is a starting point for explanation. Spikes, slow electrical potentials, and hemodynamic responses sample different aspects of neural activity, and similar timing does not establish identical content or mechanism.
Lebedev and colleagues made the distinction explicit by requiring monkeys to remember one location while attending to another. Although the task imposed a substantial short-term memory demand, the largest proportion of spatially tuned prefrontal neurons represented the attended location rather than the remembered one [@lebedevetal2004attention]. Delay activity could not be understood as storage alone. It reflected which variable currently had priority within the task.
The neural regularity is broader than the psychological category. Frontal systems remain engaged when a task relation must continue to organize behavior across an interval, whether the relation is described psychologically as memory, attention, expectancy, or preparation.
38.5 What remains effective during a delay
The word maintenance can also conceal important differences. During one delay, the system may preserve the location of an absent target. During another, it may keep a conditional rule effective, sustain attention to one sensory stream, prepare one of several possible actions, estimate when an event will occur, or retain an intermediate result that will be transformed at the next step. These variables can coexist, and a single neuron can respond to combinations of them.
The overview introduced control state for information that changes how the organism uses other information or recruits an action (Section 36.1). Here we ask what that state consists of physiologically. It may include a remembered location, a rule, or an expected outcome, but identifying its content is only part of the explanation. We must also ask how that content changes subsequent processing. A red light can mean stop, press left, compare the next two images, or ignore the next event. The visible stimulus is the same. The maintained rule changes the mapping from input to action.
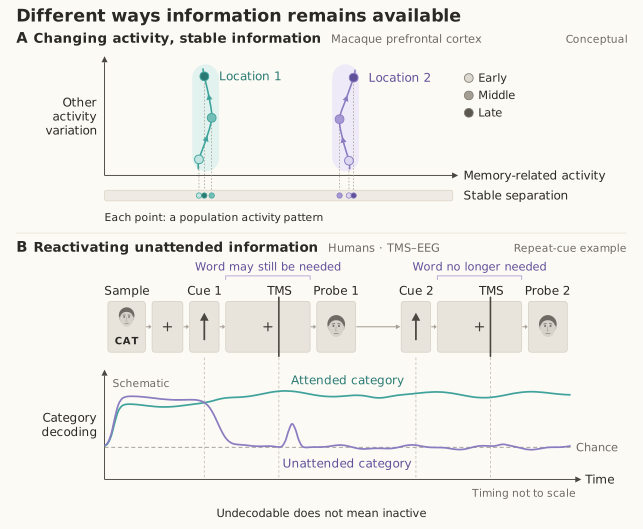
Control states need not be represented by an unchanging set of neurons firing at one rate. In monkeys using an instruction cue to determine which subsequent visual object required a response, the cue drove prefrontal populations through a sequence of states before activity settled into a relatively stable, low-activity configuration specific to the task context. When a subsequent object appeared, the population response evolved differently according to the maintained rule [@stokesetal2013dynamic]. The population changed through time while retaining information about how an upcoming object should be treated. A rule could therefore be expressed through the pattern and evolution of activity without requiring each participating neuron to remain uniformly active.
The same distinction applies to retained content. Individual prefrontal neurons can change their tuning across a delay while the population preserves a stable representation in a lower-dimensional subspace [@murrayetal2017stable]. Stability at the behavioral level therefore does not require every cellular component to remain static. An analysis can recover the remembered variable from a consistent combination of neuronal responses even while other aspects of the population change. This provides a possible readout for connected systems; decoding it does not establish that those systems use exactly that readout.
Nor must every potentially relevant item remain continuously decodable at the same strength. In human experiments, an item removed from the current focus of attention could become difficult to decode from ongoing activity and later return to an active pattern. A pulse of transcranial magnetic stimulation delivered during that latent interval briefly restored decodable information about the unattended item’s category when that item remained potentially relevant [@roseetal2016latent]. The study also found a behavioral consequence of reactivation. It supports the existence of a latent, task-dependent state; it does not directly measure a synaptic trace. Failure to decode an item from the recorded signals is not proof that all neurons representing it have stopped firing.
These findings do not replace one working-memory mechanism with another. They show why the physiological account must accommodate more than uniform persistent firing. Sustained spiking, changing population activity, and later reactivation have direct experimental support. Short-lived changes in synaptic efficacy are one proposed way of preserving latent information. These possibilities can coexist, and the evidence for their contributions differs across tasks and species.
These mechanisms bring us back to the chapter’s central question:
Temporary availability and effective control are different achievements. A neural account must explain both what information remains available and how it changes what the organism does.
38.6 Holding the line is a property of loops
The earliest delay recordings included the mediodorsal thalamus (MD). The connectional account in Section 36.5 explained why this matters: frontal cortex exchanges activity with thalamic partners while also participating in basal-ganglia and cortical circuits. Local recurrence remains important, but activity recorded in one area need not be sustained within that area alone.
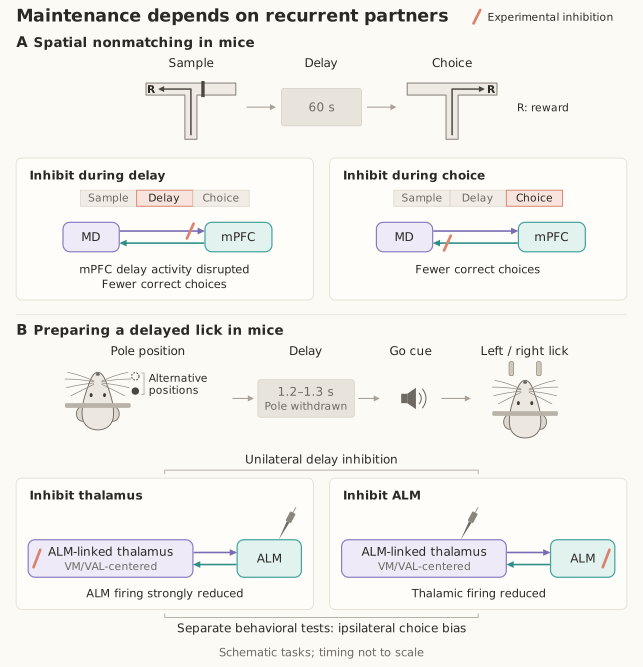
In a mouse delayed nonmatching-to-sample T-maze task, pathway-specific perturbation showed that projections from mediodorsal thalamus to medial prefrontal cortex were required during the maintenance interval, whereas the return projection from prefrontal cortex to mediodorsal thalamus contributed especially to the subsequent choice. Suppressing MD input disrupted sustained firing in delay-active prefrontal neurons, and enhancing MD excitability improved performance [@bolkan2017thalamic]. The delay-active and spatially selective populations overlapped little. Sustaining task-related activity therefore did not simply mean relaying a copy of the remembered location.
A related result emerged in mice preparing a delayed directional lick. Neurons in anterior lateral motor cortex (ALM) and connected thalamic nuclei both carried preparatory activity. Silencing either node caused activity in the other to collapse and impaired the future movement [@guoetal2017loop]. The results support maintenance through reciprocal excitation across regions. The interval-spanning state depended on the loop.
The two experiments concern different frontal territories and tasks. As Section 36.2 emphasized, mouse medial frontal cortex and ALM are not interchangeable with primate granular dorsolateral PFC. They establish a circuit principle that can be tested across systems, not a one-to-one anatomical equivalence.
Basal-ganglia circuits contribute another requirement: not every available representation should enter effective control. In a human imaging experiment, activity in prefrontal cortex and basal ganglia before a memory array predicted how effectively irrelevant items would be excluded from later representation [@mcnabklingberg2008access]. The result is often described as gating access to working memory. It supports a role in selecting what will remain influential, but the imaging association does not establish a particular cellular gate or the direction of causation. The corticostriatal and thalamic anatomy in Section 36.5 supplies candidate routes for that selection.
Posterior sensory and parietal systems carry properties of the absent stimulus and the spatial or attentional relations needed for the task. Hippocampal and medial-temporal systems can contribute when performance depends on relational or contextual information; a short delay or the presence of several items does not by itself specify their contribution. Premotor and motor systems carry prospective actions. Neuromodulatory systems alter the stability and gain of the participating populations. The overview’s D1-receptor example is relevant here: modest stimulation sharpened spatial tuning, whereas stronger stimulation degraded it [@vijayraghavan2007d1]. Modulation can change the effectiveness of a representation without specifying its content. Which partners are required depends on the task; the list is not a circuit that must be recruited in full on every trial.
The regulated body also remains inside the loop. The selected water source in the opening example does not retain a fixed value while a neutral memory system carries it forward. Section 36.4 described several routes by which bodily state influences frontal circuits. The selective-devaluation experiment in Figure 37.6 made a complementary distinction: an outcome could lose pleasantness without that change being used normally in cue-guided choice. Hypothalamic, insular, brainstem, orbital, ventromedial, and striatal signals continue to report and predict bodily state, cost, risk, and outcome. A goal can weaken because the deficit has been corrected, strengthen because the predicted heat load has increased, or be abandoned because another threat has become more consequential. Maintenance protects an expected outcome from irrelevant competition; it does not quarantine the outcome from revaluation.
The comparative evidence reinforces the functional point. In the pigeon experiment introduced in Section 36.2, learned cues signaled whether a sample would need to be remembered. Neurons in the nidopallium caudolaterale sustained activity after remember cues and reduced it after forget cues; memory was poorer when unexpectedly tested after a forget cue [@rosecolombo2005]. The avian pallium and mammalian prefrontal cortex are organized differently. Both participate in circuits that regulate whether absent information remains behaviorally available.
The control problem is therefore not exclusive to primate granular cortex. The avian comparison supports functional analogy; it does not identify the two territories as the same anatomical structure. The evolutionary continuity concerns the problem of keeping absent information useful to a body acting through time.
38.7 Stable enough to persist, flexible enough to change
The title Holding the Line can now be understood without assigning a line-holder to the brain. A task cue changes the state of a distributed controller. That state increases the influence of some representations and actions, decreases the influence of others, and persists long enough for the relevant consequence to be reached.
The central engineering problem is not maximal persistence. It is deciding which new events count as disturbances and which count as evidence that the state itself is wrong. A passing sound may be irrelevant to the route toward water. A predator on the route is not. The first should be rejected; the second should reorganize behavior.
Several operations traditionally grouped under executive function contribute to this balance, but they should not be collapsed into one faculty.
Maintenance keeps a rule, target, or expected outcome consequential after its cue disappears. Proactive control configures the system in advance so that an irrelevant stimulus or prepotent response has less influence. These operations are closely related because a strongly represented rule biases competition before conflict occurs.
Reactive stopping solves a different problem. A pending response must be cancelled when a stop signal arrives, sometimes before overt movement begins. Damage to right inferior frontal cortex impairs stop-signal performance. Functional imaging and tractography implicate a network that also includes pre-SMA and the subthalamic nucleus (STN) [@aron2003stopping; @aron2007triangulating]. The overview located these routes in relation to cortical action systems and basal-ganglia output (Section 36.6). Detecting the signal, changing priority, and suppressing a response are distinguishable contributions; these findings do not make right inferior frontal cortex a solitary brake.
Updating also differs from maintenance. New evidence must be identified as relevant, the current state must lose priority, and a replacement must gain access to control. A system that updates too readily becomes distractible. A system that updates too slowly perseverates. The two errors lie on opposite sides of the same stability–flexibility problem.
Planning can require an overarching goal to remain effective while intermediate subgoals change. This is more than keeping one item active for a longer delay. It requires monitoring progress, representing transitions, and revising the route when an intermediate prediction fails.
Initiation should remain separate again. A goal can be represented, valued, and maintained without mobilizing the organism to begin. Tomorrow Never Comes will examine apathy, abulia, and akinetic mutism precisely because making a course of action available is not the same as initiating it.
The result is not a new list of modules. It is a decomposition of control problems. The same frontal, thalamic, striatal, posterior, and motor systems can participate in several operations, but participation does not make the operations identical.
Maintained constraints usually reduce an enormous response space to actions that fit the task. In an unusual problem, that advantage can become a cost.
Reverberi and colleagues asked patients with focal lesions and healthy comparison participants to solve matchstick equations. The most difficult problems required changing the ordinary interpretation of the symbols. For the hardest problem type, 82% of the lateral frontal patients found a solution, compared with 43% of healthy comparison participants [@reverberietal2005insight].
The result does not show that lateral frontal damage improves reasoning in general. It supports a bounded tradeoff in this task. A system that strongly constrains interpretation toward normally useful representations can impede a solution that requires abandoning those representations. Stability is valuable because the world is usually structured. Flexibility is valuable because the current structure is sometimes wrong.
38.8 When a known rule loses control
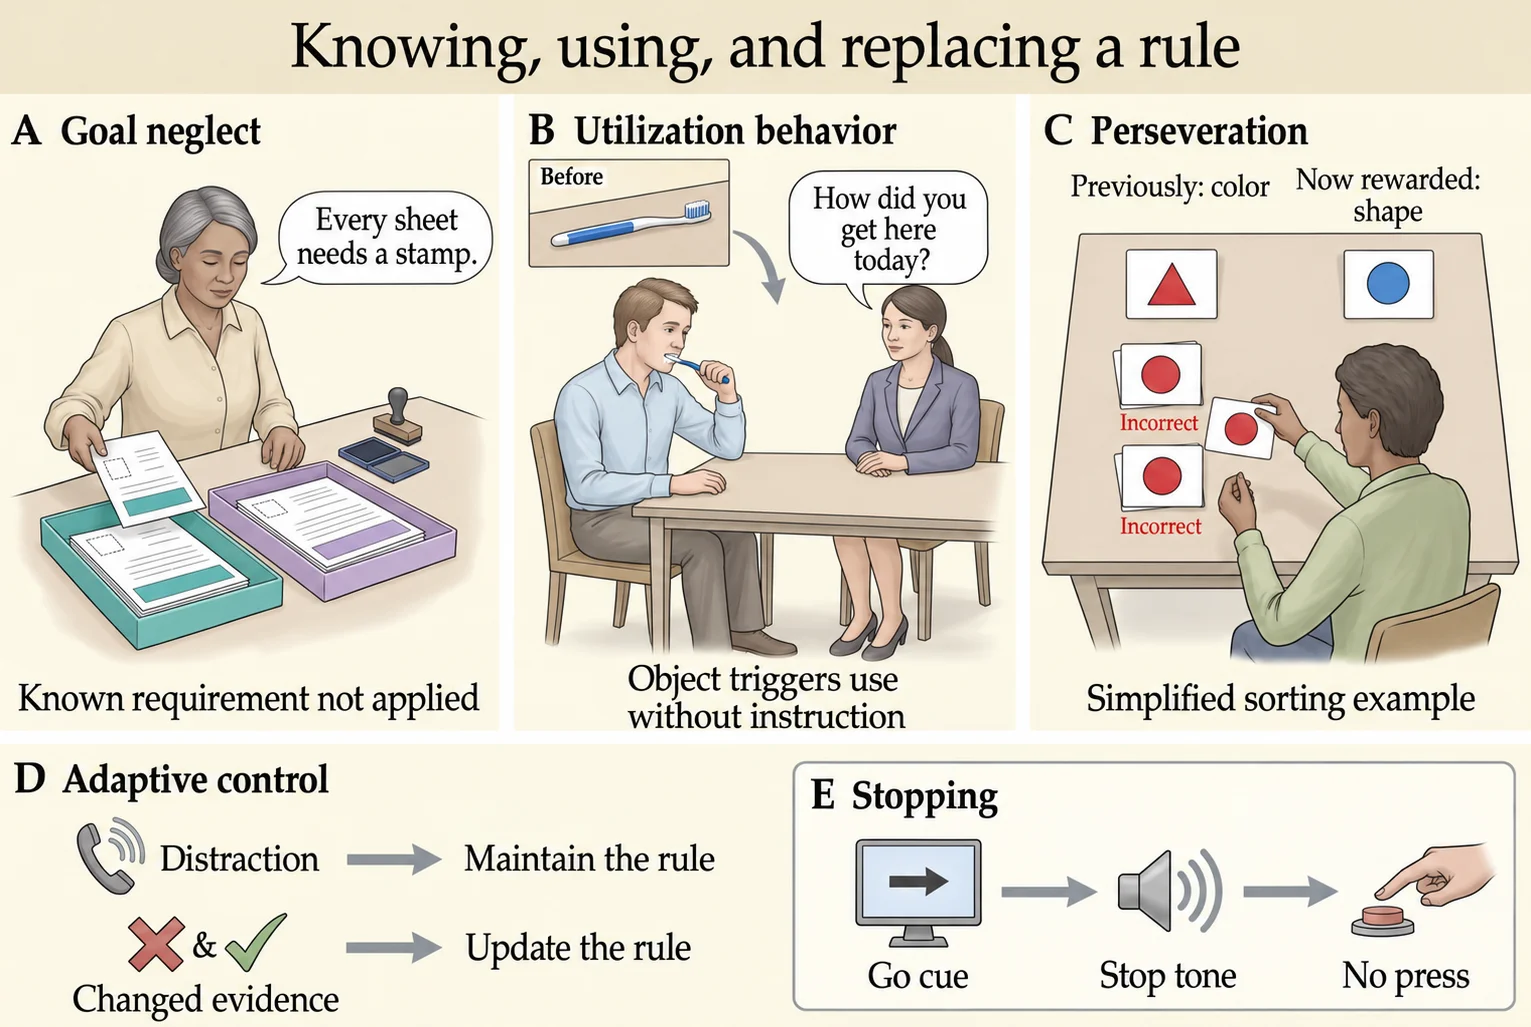
Goal neglect provides the clearest separation between possessing information and allowing that information to govern behavior. A person can understand an instruction, repeat it accurately, and then fail to implement one of its requirements when several demands must be coordinated. The rule remains available for report but drops out of effective control [@duncanetal1996goal].
This dissociation directly challenges the idea that a remembered rule is simply stored or absent. The relevant question is what the representation can do. A sentence repeated to the examiner demonstrates availability for report. Effective task control additionally requires that its content change how later events are interpreted and which actions are selected.
Novel and open-ended situations make the distinction especially visible. Shallice and Burgess described patients who performed many conventional tests adequately but failed when they had to organize several simple activities over an extended interval with little external structure [@shalliceburgess1991strategy]. The component skills were present. The patients did not reliably construct and sustain a task model that coordinated them.
Goal neglect is therefore not ordinary forgetting, and it is not evidence that one executive has disappeared. It is a failure of a known requirement to achieve or retain the neural influence needed to organize the rest of the task.
38.9 When the present gains too much control
Distraction reveals the same problem from the other side. During a delayed-response task, an irrelevant event can reorganize sensory, affective, and frontal activity strongly enough to degrade the state that supports the pending response.
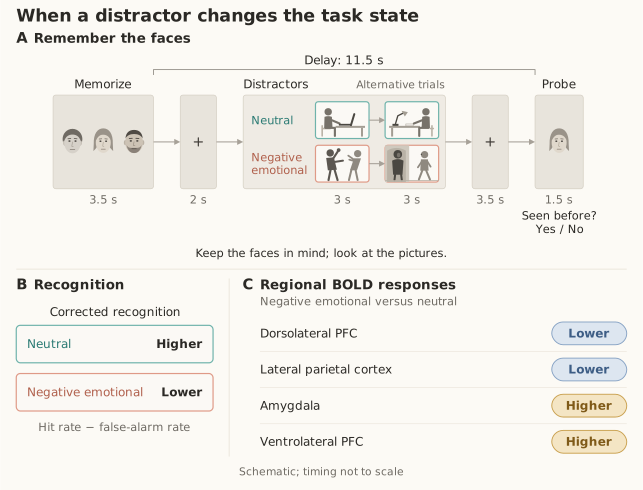
Dolcos and McCarthy presented emotional or neutral distractors during the delay of a face working-memory task. Emotional distractors impaired later performance. Negative emotional distractors elicited greater amygdala and ventrolateral prefrontal responses, together with reductions in task-sustained dorsolateral prefrontal and lateral parietal activity [@dolcosmccarthy2006interference]. The measurements reveal different responses across the participating systems. They do not establish that one ventral region directly inhibited a dorsal one, or that increased ventrolateral activity itself caused the impairment.
The distinction between value and salience developed in Chapter 37 matters here. A disturbing image can command processing because it is biologically or emotionally significant without offering a positively valued outcome. Value and salience can interact, but they are not interchangeable. An emotional event can change processing priority and interfere with the configuration required by the ongoing task.
The clinical extreme is utilization behavior. Lhermitte described patients who grasped and used objects placed before them although the objects were irrelevant to any stated goal. A comb invited combing; spectacles were put on; a glass invited drinking [@lhermitte1983utilization]. The behavior exposed an ordinary fact in exaggerated form: visible objects continuously offer actions. In intact control, those affordances compete with rules, social context, predicted outcomes, and longer-range goals. After frontal-network injury, the immediate invitation can acquire disproportionate control.
Utilization behavior should not be labeled a pure dorsolateral deficit or a simple release from one inhibitory center. The syndrome has followed different frontal and frontal-subcortical injuries, including paramedian thalamic infarction [@lhermitte1983utilization; @eslingeretal1991thalamic]. Within the account developed here, it illustrates environmental dependency: the present scene governs action more strongly than the absent variables that would normally place the scene in context.
38.10 When an old state will not release
Perseveration produces the opposite clinical appearance. The patient continues to sort, search, speak, or act according to a rule that no longer fits the evidence. The problem is not failure to maintain a control state. It is failure to replace one.
Using the Wisconsin Card Sorting Test, Brenda Milner showed a relationship between frontal lesions and difficulty shifting from one sorting principle to another [@milner1963cardsorting]. In this task, feedback reveals whether a card was sorted correctly, and the relevant principle changes without an explicit announcement. Performance therefore depends on rule discovery, feedback use, maintenance, and switching. It is not an anatomical scanner for dorsolateral prefrontal cortex. Poor performance can arise from several component failures and from damage outside one frontal territory.
The contrast with goal neglect is instructive. In goal neglect, a valid rule loses effective control. In perseveration, an invalid rule retains it. Distractibility and environmental dependency make behavior too sensitive to the present. Perseveration makes behavior insufficiently sensitive to change. No single score called executive function captures these opposed failures.
Stability and flexibility are not competing explanations of frontal function. They are the opposing demands that any temporally extended controller must regulate.
38.11 Coda: the future enters the present body
An absent future can govern action because the nervous system does not return to its pre-cue state when the cue disappears. Frontal, thalamic, striatal, posterior cortical, hippocampal, motor, and bodily systems remain configured by what the cue established. Their ongoing activity and altered interactions keep selected information, rules, priorities, and prospective actions effective across time.
Psychology describes many of these behaviors with the construct working memory. The construct is useful because temporary availability is a real feature of behavior. The physiology does not reveal a working-memory organ. It reveals multiple ways in which a distributed controller can preserve and transform variables that are absent from current input.
The control state remains open to the body. A predicted outcome can change heart rate, vascular state, visceral sensation, and readiness for action before the outcome arrives. Those anticipatory changes can in turn alter what the outcome is worth and how urgently it should be pursued. The overview’s outgoing pathways supplied routes by which a represented situation can affect bodily preparation (Section 36.6). We have followed how that situation remains effective across time; the autonomic changes and returning bodily information now deserve closer attention.
The next chapter, Feeling the Future, follows that prediction into autonomic and interoceptive state.
The evidence. Primate lateral prefrontal neurons can carry selective information across delays, and lesions of the relevant tissue impair memory-guided performance. Human electrical recordings and imaging reveal frontal participation in sustained preparation and temporary retention, while measuring different aspects of activity. Population analyses find stable information amid changing neuronal responses. Reactivation experiments reveal information that remains potentially usable when it is difficult to decode from ongoing measurements. Mouse perturbations establish causal contributions of thalamocortical interactions to maintenance in particular tasks. Clinical and behavioral studies distinguish retaining a rule, using it, resisting distraction, and replacing it.
The interpretation developed here. Working memory is a useful psychological construct whose neural realization need not be one module or mechanism. I take the recurring problem to be maintained control: selected information must remain capable of changing the organism’s next action. Lateral frontal systems participate through the differentiated connections introduced in the overview. Valuation continues while information is maintained, and the body remains part of the process. This synthesis joins findings across tasks and species without treating their circuits as interchangeable.
The open questions. How do persistent firing, changing population activity, synaptic state, and reactivation contribute under different conditions? How do recurrent circuits distinguish interference from evidence that requires updating? How does information available for report gain or lose effective control over another part of a task? And how do mechanisms studied over seconds support nested goals across minutes or longer? These questions concern both the preservation of information and the changing influence it has on behavior.